STATUS OF MARINE BIRD POPULATIONS (continued 2)
Reading edition
Nelson (1887) apparently found red-faced cormorants breeding on the Siberian and Alaskan mainlands at either side of Bering Strait, but Bailey (1948) searched for some sign of their presence and found none. Nelson (1887) also reported the red-faced cormorant from St. Matthew and St. Lawrence islands in the northern Bering Sea and from St. Michael and Nelson Island on the Alaskan coast. Gabrielson and Lincoln (1959) pointed out that it has not been found breeding north of the Pribilofs since then. Friedmann (1934) provides support for Nelson by reporting red-faced cormorant bones from archeological sites on St. Lawrence. Gabrielson and Lincoln (1959) cited two red-faced cormorants in the Leningrad Academy of Science which were collected in the Pribilofs in 1843. Dall and Bannister (1869) reported them to be plentiful on St. George Island. Baird (1869) also noted their presence in the Pribilofs.
Bent (1964) makes no mention of seeing the red-faced cormorant in the Aleutians. He gives their breeding range as the Bering Sea region, the Pribilof Islands, and perhaps the western Aleutians, the Commander Islands, and the coast of Siberia north of North Cape. The American Ornithologists' Union (1931) gave their breeding range as the Pribilof Islands, the Commander Islands, and Siberia north to North Cape.
Murie (1959) found a colony of between 4,000 and 5,000 red-faced cormorants nesting on Amak Island in 1925. In 1936 he was surprised to find that the red-faced cormorant was the most abundant breeding cormorant in the Aleutian Islands. Pelagic cormorants still appeared to be most numerous, but there were large numbers of nonbreeding birds. In 1936 he located "a good sized colony" of red-faced cormorants at Unga in the Shumagin Islands. He found about 300 birds starting their nests on 16 May.
In August 1946 Gabrielson (Gabrielson and Lincoln 1959) visited the colony at Delarof Harbor, Unga, where several thousand cormorants were observed. From a number of small samples he estimated that the red-faced cormorants outnumbered pelagic cormorants five to two. In 1973 I observed about 2,000 cormorants, mostly red-faced, in this colony. Gabrielson also located them at two other sites in the Shumagins and at Aghiyuk Island in the Semidi Islands.
Howell (1948) noted only double-crested cormorants at Double Island, Kodiak. Shortly after that the leaflet, Birds of the Kodiak Island National Wildlife Refuge (first issued in 1955), listed red-faced cormorants as common summer residents. The red-faced cormorant was next found at Katchemak Bay about 1963. Isleib (Isleib and Kessel 1973) first noticed red-faced cormorants wintering in Prince William Sound in 1969. In July 1972 Isleib and Sowl had found a colony containing 75 nests at Point Elrington at the western approach to Prince William Sound. By 1974 Isleib and Haddock (unpublished data, FWS, Anchorage, Alaska) found them east of the Copper River Delta at Wingham Island.
The relatively rapid expansion of the range and apparent population size of the red-faced cormorant is remarkable. But has this been a real expansion into vast stretches of new territory? The record in the literature which I have summarized shows, I think, something else. We can demonstrate a historical range for the red-faced cormorant that extends on the Asiatic Coast from North Cape, Siberia, south to the Kurile Islands, the entire Aleutian Arc including the Commander Islands, all the Bering Sea islands north to Bering Strait, Norton Sound, Nelson Island, and the islands south of the Alaska Peninsula at least as far east as Kodiak Island. The recently occupied coast from Cook Inlet to the Copper River may represent a real range extension. The breeding range of this species at the present time does not include parts of its historical range west of the Commander Islands or north of the Pribilof Islands.
The fragmentary record appears to show a long-term perturbation in the range and populations of the red-faced cormorant that covers at least 100 years. I believe that we are probably seeing a recovery of lost range and a return to something resembling a former distribution and abundance.
What caused the perturbation? I am not prepared to answer this question, but there are two occurrences which I find suggestive.
It is interesting to note (Dement'ev and Gladkov 1966) that on the Commander Islands the red-faced cormorant was most abundant during the first 50-odd years after the pelagic cormorants had been wiped out in the winter of 1876-77. Perhaps some clues are to be found in the interactions between these similar species.
It does not appear that the introduction of fox could have been a causative factor. The first observations of population expansion were noted almost concurrently with the heyday of the fox-farming industry. Because of its choice of nesting habitat (very steep cliffs), this cormorant would not have been affected by predators except for the one that went into a very rapid population decline at a time that would fit—the Aleut.
Jochelson (1968) and Hrdlicka (1945) summarized references to Aleut clothing in the diaries and reports of early Russian visitors to the Aleutian Islands. Evidently Aleut women sometimes wore a long, robe-like parka made of harbor seal (Phoca vitulina) skins or, for women of high rank, parkas made of sea otter (Enhydra lutra). The men in almost all reports were said to have worn bird-skin parkas; puffins and guillemots appear to have been preferred, but cormorants were sometimes used. It took about 40 puffin skins to fabricate a parka and a man evidently needed from one to three of these garments each year.
Sea otter populations were drastically reduced by Russian hunters. Rats were introduced to the Aleutians very early during the Russian period and must have had a substantial impact on populations of tufted puffins and guillemots. The introduction of fox would have had a further impact on burrow-nesting birds. Turner (1885) noted that Aleuts in the Near Islands kept the fox confined to Attu so that they could keep the fox away from the birds on Agattu. This is evidence of an Aleut recognition of serious competition. Could cormorants, particularly red-faced cormorants, have been preferred sources of fiber? Were Aleuts forced to rely more heavily on cormorant skins as puffin and guillemot numbers were reduced by rats and fox and sea otters by men?
Whatever the cause and effect, the status of red-faced cormorants now appears to be better in the Gulf of Alaska than for at least the last 100 years.
Glaucous-winged Gull (Larus glaucescens)
The glaucous-winged gull is apparently one of the more successful seabirds breeding in the Gulf of Alaska. While it is outnumbered (both locally and in total abundance) by the black-legged kittiwake, it is generally the most commonly seen and most uniformly distributed gull in the Gulf of Alaska. Murie (1959) called it the common breeding gull about the Alaska Peninsula. Cahalane (1943, 1944) considered it to be numerous to abundant around Kodiak and in the Shelikoff Strait area. Gabrielson (1944) reported that it could be seen in small numbers everywhere. Most recently, Isleib and Kessel (1973) reported it to be an abundant resident in the north Gulf Coast area. My own experience would confirm these observations.
This gull appears to use a wider variety of nesting sites than some others (Gabrielson and Lincoln 1959). Except where man's activities have created new food sources, there appears to be a close link between the location of glaucous-winged gull colonies and those of murres, kittiwakes, and cormorants. Swartz (1966) found that during the breeding season glaucous-winged gulls at Cape Thompson derived almost all of their food from murre eggs and chicks. I have noted small numbers of these gulls nesting, usually on turf near the tops of cliffs, in most colonies of favored prey species.
The glaucous-winged gull is the principal scavenger throughout much of coastal south-central Alaska. This has sometimes resulted in the development of large concentrations near canneries and, more recently, near dumps.
Two glaucous-winged gull concentrations stand out in the northern Gulf of Alaska. One of these is on Egg Island at the western end of the Copper River Delta. Patten (1976) estimated that this colony contained 10,000-12,000 gulls in 1975. At times it appears to spread onto nearby Hinchinbrook Island. M. E. Isleib (personal communication) has estimated its size as high as 25,000 gulls. The other large concentration is on the Susitna Flats across Cook Inlet from Anchorage. This colony, or colony cluster, may be larger than the one at Egg Island. There are no other known colonies even approaching these in size. Most colonies range between a few pairs and 2,000-3,000.
Glaucous-winged gulls do not appear to have had any great changes in population that can be detected from the literature. There have almost certainly been local fluctuations in the number of breeding birds as food supplies, such as canneries and dumps, have appeared or disappeared in an area. Long-term changes in salmon runs have undoubtedly had an impact as well. One other change, the reduced level of egging, has undoubtedly had an effect also. Along the Alaska Peninsula and in the Shumagin Islands, cannery workers of Filipino heritage and fishermen who have a strong Aleut heritage still harvest gull eggs for food. However, this activity is much reduced from what it must have been.
Herring Gull (Larus argentatus)
The herring gull is a resident of Upper Cook Inlet and is found up and down the coast from Prince William Sound to the Alaska Peninsula. Not too much was learned about it during the recent FWS reconnaissance. Williamson and Peyton (1963) reported the interbreeding of herring gulls and glaucous-winged gulls in this area. This interbreeding has resulted in a situation in which assignment of these gulls to one group or another in the field can be rather arbitrary. The result has most often been that field observers tend to lump them with glaucous-winged gulls unless their herring gull characteristics are obvious. Specimens collected by Williamson and Peyton (1963) indicate that herring gulls have the edge in numbers in Upper Cook Inlet.
Black-legged Kittiwake (Rissa tridactyla)
The black-legged kittiwake is the most abundant gull in the northern and western Gulf of Alaska. Colonies of this species can be found throughout the entire area, and range in size from a few pairs (Class I) to more than 100,000 birds (Class V). They may be found in essentially pure colonies, but are often found sharing colonies with murres.
The center of abundance for breeding black-legged kittiwakes in the Gulf of Alaska is in the Semidi Islands, where Palmer Sekora (U.S. Bureau of Sport Fisheries and Wildlife 1973) estimated that there were 426,000 breeding kittiwakes in 1972. He located kittiwake colonies at eight sites, ranging in size from 1,000 to 109,000 nesting birds. The size of the average colonial site was 27,000 birds. Ten sites were Class IV in size and one was a solid Class V.
The easternmost known colony in the northern Gulf of Alaska is at Wingham Island. Up to 1973, 22 colonies had been located in Prince William Sound. The largest of these contained only 5,636 nests in 1972 (Isleib and Kessel 1973). Class IV or larger colonies are found at Cape Resurrection, the Barren Islands, Chisik Island, Boulder Bay and Cape Chiniak on Kodiak Island, and at Delarof Harbor and the Haystacks in the Shumagin Islands. It is interesting to note that Gabrielson (1940) considered Whale Island to be one of the largest known kittiwake colonies in Alaska. He stated that there were many thousands of pairs extending over a mile or more of cliff. He saw a second site which he did not visit but looked equally large. A photograph in an article by East (1943) also indicated the presence of a large colony. C. J. Lensink (personal communication) estimated that there were about 100,000 kittiwakes in the colony in 1956. When last visited by Vernon Berns (personal communication), this colony contained only 3,000 birds. It is also of interest that Gabrielson (1940, 1944) did not notice either the kittiwakes or the murres now breeding on Nord Island in the Barren Islands or the kittiwakes on East Amatuli Island.
Whale Island and possibly the colonies in the Barren Islands give evidence of local population fluctuations, but for the most part I have not found an indication of a major perturbation over the past 40 years. Before 1936, the record is too fragmentary to allow an assessment.
One of the interesting aspects of kittiwake ecology in the Gulf of Alaska is the common occurrence of breeding failure. David Snarski (December 1943 Quarterly Progress Report, Alaska Cooperative Wildlife Research Unit, University of Alaska) observed breeding failure on colonies in the Tuxedni National Wildlife Refuge in 1970 and 1971 and obtained circumstantial evidence of another failure in 1972. In 1973 all of the breeding cliffs were occupied and nesting was successful. Whatever the cause of these periodic failures, they do not yet appear to have had a permanent impact that we are able to measure.
Red-legged Kittiwake (Rissa brevirostris)
Red-legged kittiwakes are not now known to breed in the western Gulf of Alaska. Turner (1886) stated that he saw a few at Sanak in 1878. We also have Stejneger's (1885) statement, that "red-legged" kittiwakes nest from Bering Island to Sanak. Friedmann (1937) reported two humeri from Kodiak Island middens. During the summer of 1976, two birds were observed off Kodiak Island by Irving M. Warner (personal communication), and one at 158°W and 54°30'-54°20'N south and east of the Shumagin Islands (Patrick J. Gould, personal communication).
Turner (1885) listed the red-legged kittiwake as abundant and breeding in the Near Islands. Turner (1886) also stated that he had seen quite a number about a cliff back of the village on Akutan Island in 1878. He added that to the westward this kittiwake was more abundant than the black-legged kittiwake. Murie (1959) expressed the opinion that Turner had confused the short-billed gull with the "short-billed" kittiwake. Clark (1911) also reported that he had seen the red-legged kittiwake in small numbers near Unalaska and that they became progressively more common west to the Near Islands. Nelson (1887) reported seeing large numbers of red-legged kittiwakes at Unalaska. Murie (1959) and Gabrielson (1940, 1944) did not see any red-legged kittiwakes in the Aleutian Islands. The species has recently been discovered breeding at Buldir and Bogoslof islands (G. Vernon Byrd, personal communication).
Is it possible that we have here another species which is exhibiting a response to some unknown long-term perturbation? The suggestion that such an event has occurred is faint, but it is there. Do we have in the red-legged and black-legged kittiwakes an example of yet another congener pair that has been affected by some perturbation in which one was affected positively and the other negatively? Clark (1911) reported small numbers of black-legged kittiwakes to go with large numbers of red-legged kittiwakes in the Near Islands, which is the reverse of the current situation.
Arctic Tern (Sterna paradisaea)
Gabrielson and Lincoln (1959) attribute to the Arctic tern the most extensive range of any Alaskan water bird. It is found in suitable habitat everywhere north of Tracy Arm in Southeastern Alaska. Murie (1959) stated that he found it nesting at suitable sites everywhere he went. Isleib and Kessel (1973) considered it to be an abundant breeder in Prince William Sound and along the northern Gulf Coast.
The Arctic tern was observed in FWS aerial surveys in Prince William Sound, and surveys in July and August 1972 provided an estimate of 45,000 terns in the Sound (Isleib and Kessel 1973). On the other hand, tern colonies were located only rarely in the FWS colony surveys before 1975. This is, however, a reflection of the equipment and methods used and not of the abundance of terns.
From the fragmentary data available, it is not possible to detect changes in Arctic tern status at the present time. We have to assume that the widespread introduction of fox had at least local impact. Although this tern uses a wide variety of nesting sites, it tends to nest on flat sites where access by mammalian predators is easy.
Aleutian Tern (Sterna aleutica)
No Aleutian tern colonies were discovered in the Gulf of Alaska area during FWS colony surveys in the early 1970's. This is again a reflection of the fact that surveys were not designed to locate tern colonies. Aleutian terns were encountered at least twice, once during late March 1972 in Hawkins Cutoff, Prince William Sound, and again when two birds were noted offshore from the Katmai National Monument on 30 May 1973 (L. W. Sowl, personal observations).
The type specimen of the Aleutian tern and a single egg were collected at Kodiak Island on 12 June 1868 by Bischoff (Coues 1874). Fisher (Gabrielson and Lincoln 1959) collected four more eggs in 1882. The bird was not found breeding there until Howell (1948) found a colony of 50 pairs at Bell's Flats in 1944. Walker (1923) found them nesting on the Situk River, Yakutat, in 1917 and shortly thereafter saw them at the Alsek River Flats. He also reported that D. H. Stevenson of the Bureau of Biological Survey had told him that they nested on the Isanotski Islands at the end of the Alaska Peninsula. This latter report was the only one from the Aleutian Island chain for many years. Isleib and Kessel (1973) considered it an uncommon local breeder in the northern Gulf of Alaska. Isleib estimated its population at a few hundred pairs on the Copper River Delta in May 1973 and 300-500 birds in June 1970. He also reported that they appeared more or less regularly near Controller Bay and off the Situk River.
In recent years Aleutian terns have been seen with increasing frequency in many places in western Alaska and the Aleutian Islands. This is probably partly due to the increasing level of field work. At Amchitka Island the several colonies that have been found in recent years are almost certainly exhibiting a response to the removal of fox from the island.
Although there is no way of determining what the past status of the Aleutian tern has been in the Gulf of Alaska area, it has been there in small numbers since it was first discovered on Kodiak. It has probably not been abundant at any time and may have suffered a long-term decline brought about by the introduction of fox.
Common Murre (Uria aalge)
The common murre is resident in the northern and western Gulf of Alaska from Pinnacle Rock, Kayak Island, westward. East of Cook Inlet colonies are located at Wingham Island, the Martin Islands, Middleton Island, Porpoise Rock in Hinchinbrook Entrance, Barwell Island/Cape Resurrection, the Chiswell Islands, the Barren Islands, and Chisik Island.
For some reason, the islands of the Kodiak-Afognak Archipelago do not host any known major murre colonies. There is also a rather large gap between the Chisik Island colony and the next major colony at Oil Creek west of Puale Bay. Directly west of Oil Creek is another colony at Cape Unalishagvak. Both of these latter colonies are Class V and they are the first colonies of this size to be encountered in the Gulf of Alaska. West of these colonies the next large colony is at Atkulik Island. To the south, midway between the last-named colonies, lies the major composite murre colony in the Semidi Islands. These sites make up the only Class VI colony in the Gulf of Alaska. Westward, the next major colony, a Class V, is at Spitz Island south of Mitrofania Island. In the Shumagin Islands one Class V colony is at Karpa Island, and lesser colonies with large murre components are found at the Haystacks, Castle Rock, and Bird Island. Only minor murre colonies are found between the Shumagin Islands and the end of the Alaska Peninsula.
Gabrielson and Lincoln (1959) were aware only of the colonies at Cape Resurrection (which Gabrielson considered to be large), at the Chiswell Islands, and at Chisik Island for the area from Cook Inlet east. Gabrielson visited the Barren Islands on 13 June 1940 and apparently did not notice the present murre colonies, both Class IV, at East Amutuli (an island which he visited) and Nord Island.
Gabrielson (Gabrielson and Lincoln 1959) found a few small colonies at Kodiak, mostly on small offshore islands. Gabrielson found common murres to be abundant in the Semidi Islands and stated that there were no notable colonies in the Shumagins, although on his return to the Shumagins in 1949 he did find a fairly large colony at the Haystacks. That size description would fit the colony that is there now. He obviously did not see the other colonies. Rausch (1958) reported murres from Middleton Island.
There is quite a difference between the distribution of murres as we know it today and the way Gabrielson and Lincoln pictured it. Why does this difference exist? There are two possible answers: either the number of colonies has increased, or the coverage of colony locations has improved. The latter case, at least, is established. I must confess to being puzzled by the way Gabrielson was able to move about close to what are now known to be sizeable colonies without seeing them, those in the Barren Islands and the Shumagin Islands in particular. Perhaps this represents the vague outlines of yet another population change.
The center of abundance for murre distribution in the Gulf of Alaska today is from Paule Bay west to eastern Shumagin Islands. The Semidi Islands are the heartland of this area of maximum abundance. We have no definitive data on species composition of these colonies. Common murres undoubtedly dominate in most of the colonies; the only ones where we know of a sizeable thick-billed murre component are in the Shumagin Islands.
Thick-billed Murre (Uria lomvia)
Thick-billed murre population information cannot be separated from that of the common murre on the basis of existing data. A direct assessment of present-day status is not possible. After reviewing what we know about their distribution, I suggest a way to examine the question indirectly.
The thick-billed murre is found in colonies with the common murre from Middleton Island westward; Rausch (1958) noted about 400 murres at Middleton Island and observed that the thick-billed murre outnumbered the common murre by several times. Isleib and Sowl (FWS, unpublished data) saw a thick-billed murre mixed with common murres at Porpoise Rock in July 1972. Isleib and Kessel (1973) expressed the opinion that small numbers of thick-billed murres will be found in most common murre colonies in the northern Gulf of Alaska when it is possible to survey these colonies in detail. Karpa Island had a significant component of thick-billed murres in June 1973, and they constituted 40% of the colony at the Haystacks (L. W. Sowl, unpublished data).
Bent (1963) reported that many thick-billed murre eggs have been taken by collectors at Round Island in the Shumagin Islands. Dall and Bannister (1869) reported a thick-billed murre that was taken at Kodiak in 1867.
The Gulf of Alaska is at the periphery of the breeding range of the thick-billed murre. While it probably occurs in mixed colonies with the common murre throughout this area, the thick-billed murre is much less abundant. Occasionally in the Gulf of Alaska, a colony will be occupied predominantly by the thick-billed murre. Gabrielson and Lincoln (1959) noted that the thick-billed murre outnumbered the common murre in many colonies in the Aleutians and that it became progressively more common at higher latitudes.
We have almost no data relative to the species composition of murre colonies in the Gulf of Alaska. Until we do it will not be possible to fully understand the population status of the thick-billed murre. It appears that changes in the species composition of murre colonies in the Bering Sea may be an indicator of perturbation. The data for the Gulf of Alaska are still too fragmentary to provide any indication of whether or not the same indicator would work there. Close monitoring of the Shumagin Islands colonies over a number of years might produce the answer.
Earlier in this paper I noted the dramatic changes in species composition of murre colonies on Walrus Island. Gabrielson and Lincoln (1959) also commented on this well-documented and anything but static situation. Investigators who visited this island during 1976 reported seeing no murres on the island and only small numbers on offshore rocks. James Bartonek (personal communication) said that this situation has prevailed for several years.
There is an indication that a similar population fluctuation and change in species composition of murre colonies have also occurred on St. Matthew Island. Bent (1963) found mostly common murres and few thick-billed murres at St. Matthew. Hanna (1916) saw only thick-billed murres. Later, Gabrielson (1941) found this to be true in 1940.
Dramatic fluctuation in murre populations may be common and, at least in some cases, the two species may be affected differently. Perhaps this phenomenon has potential for providing us with an indicator of some natural perturbations.
Peterson and Fisher (1955) expressed the opinion that thick-billed murres arrived at the nesting ledges later than the common murre and had to take the sites that were left. Tuck (1960) reported data from the western Atlantic showing that thick-billed murres arrive later than common murres. On the other hand, Belopol'skii (1961) reported data showing that the two species arrive on breeding colonies in East Murman simultaneously. At Cape Thompson, Swartz (1966) found that thick-billed murres arrived about a week before common murres. The date of arrival, while perhaps a contributing factor, is probably not decisive. Interspecific competition of another sort is indicated.
In mixed murre colonies where there are large numbers of common murres, this species occupies the choice nesting sites. Thick-billed murres are usually left with the narrower ledges while the common murres occupy the longer, broader ledges (Belopol'skii 1961). The broader ledges have lower chick and egg mortality (Spring 1971). Spring also noted that thick-billed murres are excluded from the centers of mixed colonies. Johnson (1938) found that this contributes to higher losses of eggs to predators and to the loss of other social benefits of occupying the colony center (Johnson 1941).
Kozlova (1961) said that during the occupation of a colony there is a sharp competitive struggle between the two species. In the end thick-billed murres are pushed out to the periphery of the colonies or left with narrow ledges or other equally unfavorable sites. Spring (1971) studied the functional anatomy of both species and concluded that the common murre is more successful in these encounters because it has a more upright gait and greater agility than the thick-billed murre.
It follows that in a portion of their respective ranges, where the two species overlap and where there is an equal chance that either common murres or thick-billed murres will dominate a given colony, the common murre dominates. I conclude from this that where there are dramatic changes in species composition of murre colonies, such as at Walrus Island, it is probably because the common murre has been greatly reduced in numbers at the colony.
Spring (1971) concluded that the common murre is well adapted to pursuit and capture of pelagic fishes and that the thick-billed murre is better adapted for deep diving and the capture of benthic fishes and pelagic and benthic invertebrates. Having greater latitude for food selection, the thick-billed murre would have a greater tolerance for ecological perturbations affecting the available food supply. The common murre has an advantage when pelagic fishes are available but cannot switch to the other foods as readily as can the thick-billed murre. The low density of pelagic fishes in high arctic areas probably also accounts for the greater success of the thick-billed murre at higher latitudes relative to common murres.
Belopol'skii (1961) presented data from East Murman which indicates that the common murre restricts its diet almost entirely to a small number of fish species. Swartz (1966) found strong indications that there were significant differences in the food preferences of the two species of murres. Thick-billed murres made much greater use of invertebrates. Bédard (1976) asserted that it is well known that the common murre is quite partial to zooplankton. So again the issue is not clear-cut.
The situation is, of course, much more complex than I have portrayed it. Nonetheless, I think that it offers potential for use as a tool in assessing population change and perturbations in the food supply which should be studied quite closely.
Pigeon Guillemot (Cepphus columba)
Gabrielson and Lincoln (1959) noted that the pigeon guillemot was one of the most regularly observed birds in Alaskan waters. It is found everywhere throughout the northern and western Gulf of Alaska area, with only a few understandable and relatively small blanks, such as in the silty waters of Upper Cook Inlet. Because it obviously lacks the breeding murres' need for close contact with its nearest neighbors, it is able to exploit the available nesting habitat to the fullest. It seems that literally every bit of suitable nesting habitat is normally occupied.
Because of the dispersed way in which it breeds and because it does much of its feeding in the onshore zone (which is hazardous for boats) the pigeon guillemot is an almost impossible species to inventory by standard methods.
There is no evidence that the pigeon guillemot has been greatly affected by any major perturbation. Because of its choice of nesting habitat, it is probably subject to the attack of only one egg predator, the rat. Because of its loose social structure and the way it selects nesting sites, eggs and young do not sustain loss from panic flights. Its dispersed distribution should insure that man-made impacts such as oil spills will have limited impact.
The population levels of the pigeon guillemot are probably relatively very stable. The widespread introduction of the rat to most of its nesting range undoubtedly had impact, but this impact has gone undocumented. It would be interesting to follow the response of guillemot populations on islands where rats had been totally removed, if that ever becomes more than a dream.
Marbeled Murrelet (Brachyramphus marmoratus)
The marbled murrelet apparently breeds throughout most of the northern and western Gulf of Alaska. This apparently is a necessary condition because to date, at least in this part of Alaska, we can only guess where and under what conditions this murrelet breeds.
In some relatively sheltered waters like Prince William Sound, where marbled murrelets were estimated to number about 250,000 in 1972 (Isleib and Kessel 1973), they are the most abundant seabirds. We know from Dixon (1908) and Grinnell (1910) that this has been so in Prince William Sound since the beginning of the century. We know also that the type specimens came from there as well (Stresemann 1949), which is not necessarily an indication of abundance but is suggestive of their abundance relative to species not collected.
Gabrielson (Gabrielson and Lincoln 1959) found marbled murrelets common near Yakutat, in Prince William Sound, in Resurrection Bay, and at Kodiak, and reported seeing them at the Chiswell Islands and at Chignik and Pavlof Bay on the Alaska Peninsula. Cahalane (1943, 1944) found them to be common in Kupreanof Strait, and along the Alaska Peninsula north of Katmai Bay. Murie (1959) found them all along the Alaska Peninsula. My own field notes from 1973 indicate that the only place where they were common along the Alaska Peninsula was at Wide Bay.
We can sample marbled murrelet numbers by using standard transect methodology; however, I have some very serious reservations about our ability to convert these data into a population estimate. This is not an unusual assessment for Alaskan seabirds in general, but I think it is particularly apropos to this species.
We are still able only to guess at where the marbled murrelet nests and we have not a clue as to what sort of nesting strategy they pursue. I am not prepared to accept, on the basis of one North American record (Binford et al. 1975), that tree nesting is its habit throughout its range. What has been proved is that the marbled murrelet nests in trees and not, as these authors would have us believe, that it does not nest on the ground. It has become rather fashionable to ignore the Chichagof Island record (a ground nest), but it has not been discredited. The color of the Chichagof egg differs from that of the Big Basin egg, but does agree with the one taken from an oviduct by Cantwell (Gabrielson and Lincoln 1959). My own experience leads me to believe that tree nesting, if it occurs, is not the common habit of marbled murrelets nesting in the Prince William Sound region.
After many hours of observing marbled murrelets over a period of several years, I am intrigued by a number of things. These birds, as often as not, appear to be clustered in "pairs" as they feed. This occurs even at what should be the height of the breeding season. On several occasions I have noted a very pronounced evening flight of these birds from gathering areas on the water up into the surrounding mountains at sunset. This has moved me to wonder if their nesting strategy includes incubating at night but less than full-time attendance on days when the eggs can be warmed by the sun. We know that periodic egg-neglect is an aspect of storm-petrel behavior (Pefaur 1974). Is this behavior also possible on a more regular basis in an alcid? If so, it would certainly help explain why nests are hard to find.
It is apparent that more needs to be known about the population dynamics and life history of the marbled murrelet before we can make a proper estimate of its abundance. In spite of the fragmentary record, I conclude that the marbled murrelet probably enjoys the same relative abundance and distribution that it did at the beginning of the century.
Kittlitz's Murrelet (Brachyramphus brevirostris)
The Kittlitz's murrelet is not as abundant as the marbled murrelet, but locally it is sometimes found in large numbers. FWS surveys conducted during July-August 1972 provide an estimate of 57,000 murrelets of this species in Prince William Sound. Almost a fifth of these were concentrated in Unakwik Inlet above Unakwik Reef. Even more interesting, about 2,500 of these birds were concentrated in one loose flock.
In addition to Unakwik Inlet, Kittlitz's murrelets concentrate in College Fjord in Prince William Sound and in the waters fronting the Bering-Malaspina ice-fields (Isleib and Kessel 1973). Common as they are in these waters, this species is supposed to be even more abundant at Glacier Bay. The common feature of these waters is the amount of ice that can be found below their tributary glaciers.
The Kittlitz's murrelet is apparently distributed from LeConte Bay, east of Petersburg, Alaska, north to Point Barrow and west across the Aleutians to Attu, where Murie collected a pair (Gabrielson and Lincoln 1959). I once flushed a murrelet from an area of tread and riser topography near the top of the highest point on Kiska Island in heavy cloud cover, and although I could not see this bird well, I thought it to be of this species. From the range description in Gabrielson and Lincoln (1959) and Udvardy's (1963) range map, it is apparent that the distribution of this species is rather patchy, but I suspect that for the more mountainous part of its range this is more apparent than accurate. The record is too fragmentary to allow an assessment of any change in status during the historical period.
Ancient Murrelet (Synthliboramphus antiquus)
Chase Littlejohn (Bendire 1895) spent the spring and summer of 1894 collecting eggs on islands south of the Alaska Peninsula. He has left us a detailed record of what he saw but not where he saw it. Bent (1963) stated flatly that the site of his collecting was Sanak Island and this has common acceptance. Several things in his account point to a site which was a small island with several peers close by, but this could not have been Sanak. It could have been an island in the Sanak Island group or it could equally well have been somewhere in the Sandman Reefs. Unfortunately, because of this the record is clouded. There has never been anything approaching a survey of the southern half of the Sandman Reefs. We do not know what breeding colonies are there.
At any rate, Littlejohn told of the large numbers of Leach's storm-petrels, fork-tailed storm-petrels, auklets (of which only Cassin's is specifically identified), and ancient murrelets which occupied a large number of small islands. He could not calculate the number of breeding murrelets on his small island, the size of which I interpret to have been of the same order of magnitude as two others which he estimated were about 2 acres. He does say that the murrelets must have numbered several thousand and could, if left alone by the Aleuts, have quickly grown too numerous for the island to accommodate.
Murie (1959) made a brief visit to Sanak in 1937 and learned that there were no longer any large colonies of seabirds. He attributes this to exploitation of the fisheries and to the fox-farming industry. Littlejohn told of the repeated visits of Aleuts to his small islands, where they took hundreds of birds each time and all of the eggs they could find. This kind of activity could not help but disrupt the breeding on these islands.
Littlejohn's description of the ancient murrelet's nest leaves little doubt that the birds could be reached by fox or rats with ease. The birds showed no particular care in selecting a nest site and often worked their way back no more than about a meter into the dead vegetative cover from preceding years, where they scratched out a shallow nest.
There are few records of the ancient murrelet from the northern and western Gulf of Alaska. Friedmann (1935) reported the collection of a series of eggs in 1884 on Kodiak Island. Chase Littlejohn (Bendire 1895) collected eggs from somewhere in the Sanak Group in 1894. In 1908 Dixon (Grinnell 1910) saw a bird in Port Nellie Juan. Several were seen by Jaques (1930) near Belkofski in May 1928. Gabrielson collected one bird at Cordova in September 1941 and another at the Chiswell Islands in July 1945 (Gabrielson and Lincoln 1959). He saw numerous flocks in the Gulf of Alaska on 30 July of an unnamed year. In 1943, he would have been near Cape Spencer on that date. In 1945 he would have been near the Chiswell Islands. In either case, he was probably somewhere in Blying Sound.
The ancient murrelet is relatively uncommon but regularly observed in the inshore waters along the outer coasts of the islands fronting Prince William Sound. FWS surveys in July-August 1972 provided an estimate of almost 1,000 birds, mostly in nonbreeding plumage, along the outer coast of Prince William Sound (Isleib and Kessel 1973). Small numbers were found feeding close to the Wooded Islands on 24 July (my personal observation). Rausch (1958) saw a few off Middleton Island in 1956. Isleib (Isleib and Kessel 1973) saw 400-500 widely distributed at the mouth of Yakutat Bay in July and August 1968. The only large numbers of ancient murrelets encountered on the FWS survey of the Alaskan Peninsula in 1973 were in the Shumagin Islands. They were very common in East Nagai Strait on 9 June and more than half of the 1,300 seabirds per square nautical mile encountered between Little Koniuji and Chernabura Islands on 11 June were ancient murrelets. At Nagai Island an estimated 5,000 ancient murrelets were observed in the west bay at Pirate Shake, and later (on 19 June) several were observed in the vicinity of Midun Island (FWS, Anchorage, Alaska, unpublished data).
On the basis of the observations recounted above, I have to conclude that ancient murrelets are fairly regularly, if patchily, distributed throughout the northern and western Gulf of Alaska. I do not believe that the void in their range shown for the northern Gulf of Alaska by Udvardy (1963) is correct. Several colonies are there, awaiting discovery.
Ancient murrelets are not abundant in the Gulf of Alaska but they are certainly more numerous than we have been able to prove. It is not possible to tell from the existing data whether they were once more abundant than they are now. I suspect, on the basis of the Sanak Island experience, that we can conclude that this species has been reduced in number by various of man's activities.
Cassin's Auklet (Ptychoramphus aleuticus)
Cassin's auklet is a very uncommon bird in the northern Gulf of Alaska. In the western Gulf it is more common, particularly from the Shumagins west.
This auklet apparently once bred in great numbers on islands in or near the Sanak Group where Chase Littlejohn (Bendire 1895) found them to be twice as numerous as the ancient murrelets. Murie (1959) did not find them there.
Littlejohn began encountering Cassin's auklets at sea some 290 km southeast of Unga, Shumagin Islands. Murie (1959) encountered them near the Shumagins in May 1937. During the FWS 1973 reconnaissance survey of the Alaska Peninsula, these auklets were not encountered (or at least not identified) until we reached the vicinity of Unga Strait where we saw a few in mixed flocks with other murrelets and auklets. They were most numerous in East Nagai Strait. We encountered them only twice in a situation which indicated they might be breeding—on Hall and Herendeen islands on the north end of Little Koniuji Island.
Murie (1959) considered Cassin's auklet to be no longer common west of Kodiak. In Gabrielson's many voyages through the northern and western Gulf of Alaska he encountered them only twice, once off Cape Spencer and once in the Chiswell Islands.
Thoresen (1964) commented that throughout the northern part of its range the Cassin's auklet has become gradually less frequent. Although there are no data to dispute this, I believe, as do Isleib and Kessel (1973), that they are more numerous than observations would indicate, and I would apply this to the entire area. There are certainly colonies remaining in the Shumagin Islands, and quite probably along the south coast of the Kenai Peninsula. When it is possible to fully explore the Sandman Reefs there is a good probability that they will be found there.
We can only guess at the reasons for their decline. Bendire (1895) and Murie (1959) have described some contributing factors.
Parakeet Auklet (Cyclorrhyncus psittacula)
Gabrielson and Lincoln (1959) described the parakeet auklet as the least colonial of any of the Alaskan auklets. They also considered the Aleutian Islands to be its principal nesting grounds. There are old records of breeding parakeet auklets from Kodiak (Friedmann 1935) and Little Koniuji (Bean 1882). Grinnell (1910) reported two that were seen on Green Island, Prince William Sound, and several more that were seen near Knight Island.
Murie (1959) did not see any parakeet auklets near Kodiak and Afognak islands which he considered to be the eastern part of their range. He did not think they were abundant anywhere along the Alaska Peninsula. He found a few near Sutwik Island in May 1936 and then noted that they were fairly common near the Shumagins in May 1937.
Gabrielson found this species to be quite numerous on the north side of Chowiet Island in the Semidi Islands in 1945 (Gabrielson and Lincoln 1959). He also saw numerous individuals in Marmot Strait and saw one in the Chiswell Islands during the same year. David Roseneau (Isleib and Kessel 1973) found hundreds close to East Amatuli Island in the Barren Islands in 1965.
During FWS colony surveys, parakeet auklets have been found in close proximity to six seabird colonies in Prince William Sound. During the July-August 1972 surveys, they were estimated to number about 3,000 in the Sound. They have also been found closely associated with Chisik Island (David Snarski, personal communication), the Chiswell Islands, Nord and Sud islands in the Barrens, Sea Otter Island, and Central and Long islands along the Alaska Peninsula. They were most numerous in the Shumagin Islands, where they were found near Castle Rock, Hall (9,000), Herendeen (3,000), Atkins (more than 5,000), and Little Koniuju islands. They were again encountered south and west of Cold Bay at High, Fawn, Let, Amagat, Umga, and Patton islands. Many of these islands are in the north half of the Sandman Reefs, the only portion where any attempt has been made to survey seabird colonies.
The parakeet auklet may not be abundant anywhere in the Gulf of Alaska but, based on the numbers of places it has been seen in recent years, its population appears to be well dispersed and probably doing very well. This auklet is most abundant from the Shumagin Islands westward. It is almost certainly more numerous than has been thought. Its habits are secretive enough so that it could easily escape notice.
Because the parakeet auklet nests predominantly under boulders, it probably was not much affected by fox. Rats would certainly have reduced its numbers wherever these were introduced into its breeding habitat. We have no data to tell us whether there may have been population fluctuations in the past, but there undoubtedly were at least minor ones locally after rats were introduced.
Crested Auklet (Aethia pygmaea)
Udvardy (1963) shows the breeding range of the crested auklet as extending from southern Kodiak Island westward. Within the northern and western Gulf of Alaska, it is certainly most abundant in the eastern Shumagin Islands.
Isleib saw this auklet in Prince William Sound 3 times during the winter of 1972-73. These are the only records he was aware of for that area (Isleib and Kessel 1973). David Roseneau (Isleib and Kessel 1973) saw several in Amatuli Cove, Barren Islands, in June 1965. I observed one in the vicinity of Cape Spencer in August 1973.
Friedmann (1935) listed the crested auklet as a breeding bird at Kodiak, but considered it to be much more abundant as a wintering bird. Townsend (1913) has provided us with a vivid description of the myriads of crested auklets he encountered at Yukon Harbor, Little Koniuji Island. Gabrielson and Lincoln (1959) noted large numbers of crested auklet around Simeonof and Bird islands in the Shumagin Islands in 1946 and stated that the Yukon Harbor colony was still thriving.
Crested auklets were not encountered on the 1973 FWS reconnaissance survey until we reached the Shumagin Islands. They were abundant only at the southeastern end of Little Koniuji, where we encountered perhaps 10,000 in Yukon Harbor and more than 50,000 in a small cove directly south of Yukon Harbor on the opposite side of the island. As numerous as they were, they did not match Townsend's myriads or even come close to his assessment that they "were here more numerous than the 'choochkies' at St. George." St. George Island in the Pribilofs is famous for its least auklets which, in the past, have been estimated to number as high as 36 million (Peterson and Fisher 1955). The numbers there today do not even approach this level and we have no way of knowing how abundant they were when Townsend visited the Pribilofs, but I think it is safe to say that they probably numbered in the millions. There are probably more crested auklets than we observed on Little Koniuji, but there is certainly no longer anything approaching millions of birds. Properly pronounced, Koniuji is the Aleut name for the crested auklet, so we can assume that the original inhabitants were impressed by its numbers.
During the 1973 FWS survey we did not see crested auklets at either Simeonof or Bird islands. On the overgrazed and cattle-trampled Simeonof it does not seem possible that any could still exist.
I suspect that a cattleman's greed has been the undoing of any crested auklets that may have nested on Simeonof Island. This would not account for the loss of any colonies that may have been on Bird Island, but the decaying fox-trapper's cabin on that island undoubtedly tells the story. Churnabura, with its feral cattle, presents much the same problem as Simeonof. As for Little Koniuji, have horned puffins been partly responsible for the decrease in crested auklets? The puffin colony at the south end of Little Koniuji must be exactly where Townsend's millions of crested auklets once nested.
Least Auklet (Aethia pusilla)
No least auklets were encountered in FWS surveys in the Gulf of Alaska in the early 1970's. Udvardy (1963) shows their breeding range as starting well west in the Aleutians. Gabrielson and Lincoln (1959) give the eastern limit of their breeding range as the Shumagin Islands. Bent (1963) listed their breeding range as extending east to Kodiak Island, and Friedmann (1935) knew of only a few specimens taken in the winter from Kodiak. Perhaps least auklets nested somewhere in the western Gulf of Alaska, and they may still, but at the moment we have no evidence to prove that they do.
Rhinoceros Auklet (Cerorhinca monocerata)
Udvardy (1963) would have us believe that the rhinoceros auklet did not nest between southeastern Alaska and the southern Kurile Islands. Bent (1963b), on the other hand, lists their breeding range as extending from Washington to Agattu. Clark (1910) noted this species in small numbers at Atka and Agattu. Because of the lack of proof, Udvardy probably had no options. I believe that Bent was probably closer to describing their original range. I base this assumption on recent observations and on the additional fragments of information reported by Gabrielson and Lincoln (1959). Murie (1959) failed to find this species anywhere in the Aleutians, but his primary reason for being there, the fox-farming industry, may have had a lot to do with his not being able to find any.
The FWS surveys in Prince William Sound in July-August 1972 located small numbers of rhinoceros auklets in breeding plumage at the Wooded Islands and at Stoney Island and Channel Island in Montague Strait. These birds gave every impression of being local breeders. David Roseneau (Isleib and Kessel 1973) encountered two at the Barren Islands in June 1965. Isleib and Kessel (1973) list a few other records from this area.
My own experience leads me to believe that there is a large colony somewhere on Afognak Island, probably on or near Tonki Cape. On 30 May 1973 I noted a lone bird north of Afognak Island. Later, on 8 and 9 August, I saw several in the same area. On 13 August in Marmot Strait I observed a number of rhinoceros auklets, either singly or in groups of up to 12. Some of these had small fish in their beaks. As they flushed, they all flew off toward Tonki Cape. This observation was made just at last light, and I believe that there were many others about that could not be seen in the dying light. We did not encounter this species along the Alaska Peninsula during the FWS survey in 1973 until we reached the end. There I had one quick glimpse of what I was certain was a rhinoceros auklet at Amagat Island.
Horned Puffin (Fratercula corniculata)
The horned puffin is one of the most abundant breeding birds in the Gulf of Alaska. There are only a few really large colonies but these birds breed just about anywhere there is a cliff (even a low one) with suitable fractures and crevices. During the Alaska Peninsula surveys in 1973, I estimated that the frequency with which these birds were seen on the water was about half that of the tufted puffin. They have been recorded in so many places that there is nothing to be gained by a reiteration of the record in the literature.
The horned puffins reach their greatest density in the Gulf of Alaska west of Kodiak Island. Murie (1959) estimated that the colony at Amagat Island, Morzhovi Bay, contained 15,000 birds, one of the largest he had seen. It contained at least 50,000 in 1973. Even at that, it was no match for the colony on Little Koniuji Island with its minimum 140,000 horned puffins. Other colonies with large horned puffin components were at High Island (40,000), Castle Rock (20,000), Mitrofani Island (35,000), and Sosbee Bay (15,000).
Earlier in this paper, I commented at length on the great and often rapid fluctuations in populations of tufted puffins. The same phenomenon affects horned puffins. In 1975 there were relatively small numbers of horned puffins at Little Koniuji where they had flourished 2 years earlier (James Bartonek, personal communication). Because they are apparently subject to erratically oscillating populations, it is hard to tell how they have fared over the years.
Tufted Puffin (Lunda cirrhata)
The tufted puffin, as previously indicated, is also a bird with widely fluctuating populations. Until we develop an understanding of their population dynamics and can understand the underlying cause of these fluctuations it will not be possible to assess trends in their populations or understand the implications of such trends.
Tufted puffins are abundant throughout the Gulf of Alaska. Small colonies can be located almost anywhere. Along the Alaska Peninsula there are a number of colonies with an estimated breeding population in 1973 of more than 15,000 birds. These are: Ashiiak Island (20,000), Central Island (90,000), the Brother Islands (45,000), The Haystacks (19,000), Castle Rock (85,000), Bird Island (none, but may contain 500,000-1,000,000 at times), Peninsula Islands (35,000), the Twins (18,000), Amagat Island (40,000), and Umga Island (22,000). These colonies correspond to the area where colonies were listed for the horned puffin.
Tufted puffin populations respond readily to some undetermined short-term perturbations. This is clearly demonstrated by their rapid population fluctuations. Because of their numbers and because of the apparent rapidity with which their numbers rebound, it is not so apparent that they have been affected by long-term perturbations, as so many other seabirds apparently have.
There is much unused or underused nesting habitat suitable for this species. In some cases there are very strong clues pointing to why this habitat is vacant. On many islands along the Alaska Peninsula, which have very good-looking tufted puffin nesting habitat and no puffins, there are visible signs of the presence of fox—either fox trails or abandoned trappers' cabins. I also suspect that the brown bear (Ursa arctos) is another possible contributing factor to population declines of burrow nesters along this coast. I have seen brown bears swimming from island to island on foraging expeditions. George J. Divoky (personal communication) has found brown bears visiting Ugaiushak Island, which is 13 km from shore. There are other islands between Ugaiushak and the mainland but the shortest route from shore would require one swim of 7 km. The motivation must be strong.
Tufted puffins may shift from colony to colony. This could be an explanation for apparent local population fluctuation, but if so, I am puzzled by the apparent tenacity with which puffins cling to some sites. Their constant occupancy of sites where the vegetative mat is breakaway tundra (Amundsen 1972) or is underlain by sand results in the destruction of these sites. Tufted puffins often cling to them in spite of the fact that they have been reduced to "slums."
My conclusion is that in spite of their large numbers it appears that tufted puffin populations in the Gulf of Alaska probably have been reduced to a level below that of their undisturbed state.
Conclusions
Seabird numbers in the Gulf of Alaska are not static. Generally, they are probably much less abundant than they were when Bering made his voyage of discovery. There are, nonetheless, considerable numbers of seabirds breeding along the coasts of these waters. Some species show signs of recovery from past insults by man. With enlightened management there is still time to preserve the vast natural heritage that they represent and, in many cases, to improve their status.
In attempting to address a complicated subject in short space and a relatively narrow frame of reference, I have certainly erred a number of times. I would like to see the wealth of new data that will be derived from current work applied to this concept. An understanding of past population fluctuations and the underlying perturbations that they reflect is essential for managers faced with the problem of making good decisions on measures to mitigate the potential adverse impact of development.
References
American Ornithologists' Union. 1931. Check-list of North American birds, 4th ed. American Ornithologists' Union, Baltimore, Md. 530 pp.
American Ornithologists' Union. 1957. Check-list of North American birds, 5th ed. American Ornithologists' Union, Baltimore, Md. 691 pp.
Amundsen, C. C. 1972. Plant ecology of Amchitka Island. Amchitka bio-environmental program. Final Report, Battelle Columbus Lab., Columbus, Ohio. 27 pp.
Bailey, A. M. 1948. Birds of arctic Alaska. Colo. Mus. Nat. Hist. Pop. Publ. 8. 316 pp.
Baird, S. F. 1869. On additions to the bird fauna of North America, made by the scientific corps of the Russo-American Telegraph Expedition. Trans. Chic. Acad. Sci. 1(2):311-325.
Beaglehole, J. C. 1974. The life of Captain James Cook. Stanford Univ. Press, Stanford, Calif. 734 pp.
Bean, T. H. 1882. Notes on birds collected during the summer of 1880 in Alaska and Siberia. Proc. U.S. Natl. Mus. 5:144-173.
Bédard, J. 1976. Coexistence, coevolution and convergent evolution in seabirds: a comment. Ecology 57(1):177-184.
Belopol'skii, L. O. 1961. Ecology of sea colony birds of the Barents Sea. (Transl. from Russian.) Israel Program for Scientific Translations, Jerusalem. 346 pp.
Bendire, C. 1895. Notes on the ancient murrelet (Synthliboramphus antiquus) by Chase Littlejohn with annotations. Auk 12(3):270-278.
Bent, A. C. 1963. Life histories of North American diving birds. Dover Publications, Inc., New York. 239 pp.
Bent, A. C. 1964. Life histories of North American petrels, pelicans and their allies. Dover Publications, Inc., New York. 335 pp.
Binford, L. C., B. G. Elliot, and S. W. Singer. 1975. Discovery of the nest and downy young of the marbled murrelet. Wilson Bull. 87(3):303-319.
Bowles, J. H. 1908. Tapeworm epidemic among Washington seabirds. Condor 11:33.
Cahalane, V. H. 1943. Notes on the Kodiak-Afognak Island group. Auk 60(4):536-541.
Cahalane, V. H. 1944. Birds of the Katmai region, Alaska. Auk 61(3):351-375.
Clark, A. H. 1910. The birds collected and observed during the cruise of the United States Fisheries Steamer "Albatross" in the North Pacific Ocean and in the Bering, Okhotsk, Japan and Eastern seas from April to December 1906. Proc. U.S. Natl. Mus. 38:25-74.
Cody, M. L. 1973. Coexistence, coevolution and convergent evolution in seabirds. Ecology 51(1):31-44.
Coues, E. 1874. Birds of the Northwest. U.S. Geological Survey of the Territories, Misc. Publ. 3. 791 pp.
Dall, W. H. 1873. Notes on the avifauna of the Aleutian Islands, from Unalaska eastward. Proc. Calif. Acad. Sci. 5(1):25-35.
Dall, W. H. 1874. Notes on the avifauna of the Aleutian Islands, especially those west of Unalaska. Proc. Calif. Acad. Sci. 5:270-281.
Dall, W. H., and H. M. Bannister. 1869. List of the birds of Alaska, with biographical notes. Trans. Chic. Acad. Sci. 1(2):267-310.
Dement'ev, G. P., and N. A. Gladkov, eds. 1966. Birds of the Soviet Vol. I. (Transl. from Russian.) Israel Program for Scientific Translations, Jerusalem. 553 pp.
Dixon, J. S. 1908. Field notes from Alaska. Condor 10:139-143.
East, B. 1943. Seabird cities of the Aleutians. Nat. Hist. 51:64-71.
Fisher, J., and R. M. Lockley. 1954. Seabirds. William Collins and Sons, London. 320 pp.
Friedmann, H. 1934. Bird bones from Eskimo ruins on St. Lawrence Island. J. Wash. Acad. Sci. 24:83-96.
Friedmann, H. 1935. The birds of Kodiak Island, Alaska. Bull. Chic. Acad. Sci. 5(3):13-54.
Friedmann, H. 1937. Bird bones from archeological sites in Alaska. J. Wash. Acad. Sci. 27:431-438.
Gabrielson, I. N. 1940. America's greatest bird concentrations, Part I. Bird Lore 42:497-506.
Gabrielson, I. N. 1941. America's greatest bird concentrations, Part II. Audubon Mag. 43:15-23.
Gabrielson, I. N. 1944. Some Alaskan notes. Auk 61:105-130, 207-287.
Gabrielson, I. N., and F. C. Lincoln. 1959. The birds of Alaska. The Stackpole Company, Harrisburg, Penn. 922 pp.
Golder, F. A. 1925. Bering's voyages, Vol. II. American Geographical Society No. 2. 290 pp.
Grinnell, J. 1910. Birds of the 1908 Alexander Alaskan Expedition with a note on the avifaunal relationships of the Prince William Sound district. Univ. Calif. Publ. Zool. 5:361-428.
Hanna, G. D. 1916. Records of birds new to the Pribilof Islands, including two new to North America. Auk 33:400-403.
Howell, J. C. 1948. Observations on certain birds of the region of Kodiak Island. Auk 65:352-358.
Hrdlicka, A. 1945. The Aleutian and Commander Islands and their inhabitants. Wistar Institute Anatomical Biology, Philadelphia. 630 pp.
Isleib, M. E., and B. Kessel. 1973. Birds of the North Gulf Coast-Prince William Sound region, Alaska. Biol. Pap. Univ. Alaska No. 14. 148 pp.
Jaques, F. L. 1930. Water birds observed on the Arctic Ocean and the Bering Sea in 1928. Auk 47:353-366.
Jochelson, W. 1968. History, ethnology and anthropology of the Aleut. Carnegie Inst. Wash. Publ. 432. 91 pp.
Johnson, R. A. 1938. Predation of gulls in murre colonies. Wilson Bull. 50(3):161-176.
Johnson, R. A. 1941. Nesting behavior of the Atlantic murre. Auk 58(2):152-163.
Kozlova, E. V. 1961. Charadriiformes, Suborder Alcae. Fauna of USSR: Birds 2:1-140. (Transl. from Russian.) Israel Program for Scientific Translations, Jerusalem. 140 pp.
Lockley, R. M. 1962. Puffins. The Natural History Library, Anchor Books, Doubleday and Company, Inc., Garden City, N. Y. 222 pp.
Murie, O. J. 1959. Fauna of the Aleutian Islands and the Alaska Peninsula. U.S. Fish Wildl. Serv., N. Am. Fauna 61. 406 pp.
Nelson, E. W. 1887. Report upon natural history collections made in Alaska between the years 1877 and 1881. U.S. Army Signal Corps. Arct. Ser. Pub. 3.
Nichols, J. T. 1927. Tubinares of the Northwest Coast. Auk 44(3):326-328.
Orth, D. J. 1967. Dictionary of Alaska place names. Geol. Surv. Prof. Pap. 567. 1084 pp.
Palmer, R. S. 1962. Handbook of North American Birds. Vol. I. Yale University Press, New Haven, Conn. 567 pp.
Patten, S. M., Jr. 1976. Sympatry and interbreeding of herring and glaucous-winged gulls in southern Alaska. Pac. Seabird Group Bull. 3(1):25-26.
Pefaur, J. E. 1974. Egg-neglect in the Wilson's storm petrel. Wilson Bull. 87(1):16-22.
Peterson, R. T., and J. Fisher. 1955. Wild America. Weather Vane Books, New York. 434 pp.
Rausch, R. L. 1958. The occurrence and distribution of birds on Middleton Island, Alaska. Condor 60:227-242.
Schlegel, H. 1862-64. A catalogue of birds in the Dresden Museum of Natural History, Leyden. Dresden Museum of Natural History, 7 Vols.
Sowl, L. W., and J. C. Bartonek. 1974. Seabirds—Alaska's most neglected resource. Trans. N. Am. Wildl. Natl. Resour. Conf. 39:117-125.
Spring, L. 1971. A comparison of functional and morphological adaptions in the common murre (Uria aalge) and thick-billed murre (Uria lomvia). Condor 73:1-27.
Stejneger, L. 1885. Results of ornithological explorations in the Commander Islands and in Kamtschatka. Bull. U.S. Natl. Mus. 29:1-382.
Stresemann, E. 1949. Birds collected in the North Pacific area during Captain James Cook's last voyage (1778 and 1779). Ibis 91:244-255.
Swartz, L. G. 1966. Sea-cliff birds. Pages 611-678 in N. J. Wilimovsky and J. N. Wolf, eds. Environment of the Cape Thomson Region, Alaska. U.S. Atomic Energy Commission, Oak Ridge, Tenn.
Thoresen, A. C. 1964. The breeding behavior of the Cassin's auklet. Condor 66:456-476.
Townsend, C. H. 1913. The crested auklet. Bird-Lore 15:133-136.
Tuck, L. M. 1960. The Murres. Queen's Printer, Ottawa. 260 pp.
Turner, L. M. 1885. Notes on the birds of the Near Islands, Alaska. Auk 2:154-159.
Turner, L. M. 1886. Contributions to the natural history of Alaska. Part V, Birds. U.S. Army, Signal Corps, Washington, D.C. Pages 115-196.
Udvardy, M. D. F. 1963. Zoogeographic study of the Alcidae. Pages 85-111 in J. L. Gressitt, ed. Pacific Basin biogeography, a symposium. Pac. Sci. Congr. Proc. 10.
U.S. Bureau of Sport Fisheries and Wildlife. 1973. Semidi Islands wilderness report. Semidi Islands, National Wildlife Refuge. (Unpublished report)
U.S. Department of Commerce. 1964. United States Coast Pilot, No. 9, Pacific and Arctic Coasts, Cape Spencer to the Beaufort Sea. Coast and Geodetic Survey, Washington, D.C. 330 pp.
Walker, E. P. 1923. Definite breeding record for the Aleutian tern in southern Alaska. Condor 25:113-117.
Willet, G. 1914. Birds of Sitka and vicinity, Southeastern Alaska. Condor 16:71-91.
Willet, G. 1918. Bird notes from Forrester Island, Alaska. Condor 20:85.
Williamson, F. S. L., and L. S. Peyton. 1963. Interbreeding of glaucous-winged herring gulls in the Cook Inlet Region, Alaska. Condor 65:28.
Status and Distribution of Breeding Seabirds of Southeastern Alaska, British Columbia, and Washington
by
David A. Manuwal
College of Forest Resources University of Washington Seattle, Washington 98195
and
R. Wayne Campbell
Provincial Museum Victoria, British Columbia, Canada
Abstract
Current breeding seabird population estimates, nest-site preferences, and population changes are reviewed for southeastern Alaska, British Columbia, and Washington. There are 19 species of seabirds and a minimum of 216,566 pairs breeding in British Columbia and Washington. There are limited data on breeding populations for southeastern Alaska. Species diversity ranges from 17 species in Alaska to 15 species in British Columbia and 14 species in Washington. Eighty percent of all British Columbia seabirds breed on the east coast of Queen Charlotte Islands and the northwest coast of Vancouver Island. The three most numerous species in British Columbia are the fork-tailed storm-petrel, Oceanodroma furcata (31.3%); Cassin's auklet, Ptychoramphus aleuticus (24.6%); and ancient murrelet, Synthliboramphus antiquus (12.5%). In Washington, 74% (43,274 pairs) of the seabird population resides on the Olympic coast; the remaining 26% are in the San Juan Island area. About 54% of this population consists of the common murre (Uria aalge) and rhinoceros auklet (Cerorhinca monocerata). The rhinoceros auklet and glaucous-winged gull (Larus glaucescens) make up 97% of the total seabird population of the San Juan Islands. About 68% of all seabirds on the northeastern Pacific coast are nocturnal, burrow or rock crevice-nesting species. Currently available population data are inadequate to determine significant changes in population density for most species. Suggested topics for future research are presented.
The purpose of this paper is to discuss the known distribution, habitat, abundance, and status of breeding seabirds of the Alexander Archipelago in southeastern Alaska, the Province of British Columbia, Canada, and the State of Washington.
Even though several studies of the breeding biology of several seabird species in this area have been published, there have been few published surveys of known breeding colonies. In British Columbia the most extensive work has been done by the British Columbia Provincial Museum and the University of British Columbia (Drent and Guiguet 1961). Gabrielson and Lincoln (1959) summarized the available literature on Alaskan birds up to about 1958. Since then, no extensive surveys have been conducted in southeastern Alaska. The U.S. Department of the Interior (1972), in its environmental impact statement for the Trans-Alaska Pipeline, presented additional information on the seabirds of other parts of Alaska. In Washington, there are no published comprehensive surveys except those of Kenyon and Scheffer (1961) and unpublished surveys by the U.S. Fish and Wildlife Service and the University of Washington.
Table 1.
Taxonomic distribution of marine birds breeding along the Pacific Coast of Washington, British Columbia, and southeastern Alaska.
Family Common name Regions
British Columbia Washington Southeastern Alaska Total forms
Hydrobatidae Storm-petrels 2 2 2 2
Phalacrocoracidae Cormorants 3 3 1 3
Haematopodidae Oystercatchers 1 1 1 1
Laridae Gulls and terns 2 2 3 4
Alcidae Auks, murres, puffins 6 7 9 9
Total 14 15 16 19
Taxonomic Distribution of Marine Birds
There are 19 species of seabirds that breed along the Pacific coast of southeastern Alaska, British Columbia, and Washington (Table 1). Southeastern Alaska has the largest number (17) of species. Errors in species identification are most likely with the Larus gulls, particularly in southeastern Alaska where the herring gull (L. argentatus) and glaucous-winged gull (L. glaucescens) breed in mixed colonies (Patten and Weisbrod 1974). A similar situation exists in Washington where the western (L. occidentalis) and glaucous-winged gulls intergrade (Scott 1971). Brandt's (Phalacrocorax penicillatus) and double-crested cormorants (P. auritus) are often difficult to identify from the air. This would be a problem in Washington and the southwest coast of Vancouver Island, where the two species are locally sympatric.
Southeastern Alaska
The area under consideration is the 400-km-long Alexander Archipelago (Fig. 1). This complex pattern of islands, bays, and inlets is characterized by extremely high precipitation and typical cool marine temperatures. Average annual precipitation in the Sitka area is 245.4 cm (1931-60), and the average annual temperature is 6.3°C (U.S. Weather Bureau 1974). As a consequence of this cool, humid environment, most of the islands are densely covered with conifers, chiefly Sitka spruce (Picea sitkensis) and hemlock (Tsuga heterophylla), and an almost impenetrable shrub cover composed of salmonberry (Rubus spectabilis), elderberry (Sambucus callicaipa), devil's club (Echinopanax horridus), and three species of Vaccinium (Heath 1915).
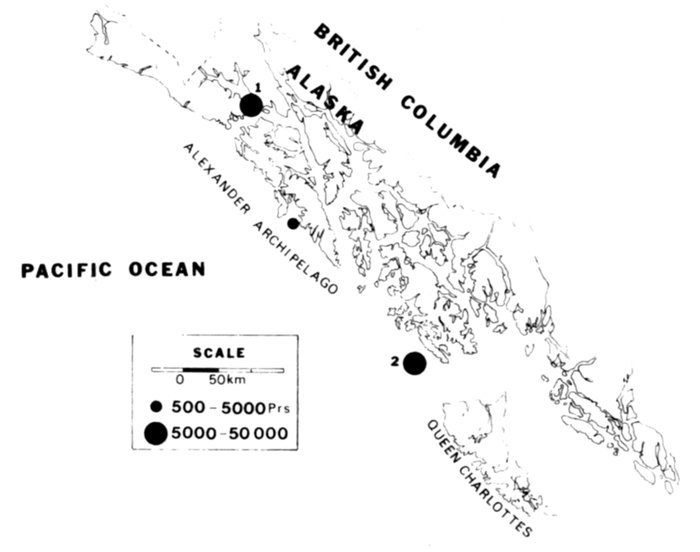
Fig. 1. Map of southeastern Alaska showing major seabird breeding colonies: 1—North Marble Island; 2—Forrester Island.
There are 16 species of marine birds breeding in the Alexander Archipelago. The major seabird breeding colonies are located at Glacier Bay and at St. Lazaria, Hazy, and Forrester islands (Fig. 1; Table 2). Published surveys of these colonies are available only for St. Lazaria (Willett 1912) and Forrester islands (Heath 1915; Willett 1915). Several authors have reported on seabirds from surrounding areas (Grinnell 1897, 1898, 1909; Swarth 1911, 1922, 1936; Patten 1974). There have been no surveys of seabirds of southeastern Alaska since before the 1940's (J. G. King, Jr., personal communication). However, since census data are available for only two colonies, we discuss them in more detail.
Table 2.
Population estimates of seabirds breeding on St. Lazaria and Forrester islands, southeastern Alaska
(data from Willett 1912 and 1915).
Bird species St. Lazaria Island Forrester Island
Number of pairs Percent of total Number of pairs Percent of total
Fork-tailed storm-petrel 2,000 8.0 10,000 6.0
Leach's storm-petrel 20,000 80.0 50,000 30.0
Pelagic cormorant 150 0.6 150 0.0
Black oystercatcher 4 0.0 50 0.0
Glaucous-winged gull 300 1.2 8,000 4.8
Herring gull 220 0.0
Common murre 300 1.2 20,000 12.0
Pigeon guillemot 150 0.6 300 0.0
Ancient murrelet 20,000 12.0
Cassin's auklet 2,000 1.2
Rhinoceros auklet 75 0.0 20,000 12.0
Horned puffin 12 0.0 1,100 0.7
Tufted puffin 2,000 8.0 35,000 21.0
Total 24,991 166,820
The studies by Willett (1912, 1915) and Heath (1915) provide some base-line information on species composition and abundance with which future studies on St. Lazaria and Forrester islands can be compared (Table 2). The somewhat greater species diversity on Forrester Island is primarily due to its greater size and more suitable soil type for ancient murrelets (Synthliboramphus antiquus) and Cassin's auklets (Ptychoramphus aleutica), species that are absent on St. Lazaria. Storm-petrels (Oceanodroma spp.) are the most numerous species on both islands, but there are proportionately more storm-petrels (88%) on St. Lazaria than on Forrester (36%). On the other hand, there are many large, burrowing alcids on Forrester Island. Nearly a third of the birds on Forrester are rhinoceros auklets (Cerorhinca monocerata), tufted puffins (Lunda cirrhata), and horned puffins (Fratercula corniculata).
The species composition of seabirds breeding on other islands is similar to that found on Forrester and St. Lazaria islands but less abundant. In Glacier Bay, for example, the only population data available are those provided by Patten (1974) for North Marble Island: pelagic cormorants, Phalacrocorax pelagicus (30 pairs); black oystercatchers, Haematopus bachmani (8); herring gulls (7); glaucous-winged gulls (500); common murres, Uria aalge (18); pigeon guillemots, Cepphus columba (60); horned puffins (4); and tufted puffins (30).
At the present time, it is impossible to draw any conclusions about changes in population density and distribution for most of the seabirds breeding in southeastern Alaska. Adequate data are available only for St. Lazaria and Forrester islands where Willet and Heath provided the only early extensive census data for this part of Alaska.
British Columbia
The rugged British Columbia coastline is characterized by 930 km of islands and inlets (Figs. 2, 3). With the exception of the inner southern portion, this coast is mostly uninhabited. The physical characteristics of the offshore islands are similar to those found off the Washington coast. Descriptions of some of these islands and the 15 species of breeding seabirds on them have been given by Drent and Guiguet (1961), Guiguet (1971), and Summers (1974).
A detailed analysis of British Columbia seabirds is not presented here since a more thorough analysis is in preparation by R. W. Campbell and R. H. Drent (manuscript). Instead, we present seabird population estimates available for the Province up to the summer of 1975; Tables 3 and 4 summarize these estimates for the five major portions of coastal British Columbia. The coast of British Columbia contains a myriad of small islands where there may be small numbers of breeding seabirds. Many of these have not been censused and are too numerous to include in Tables 3 and 4.
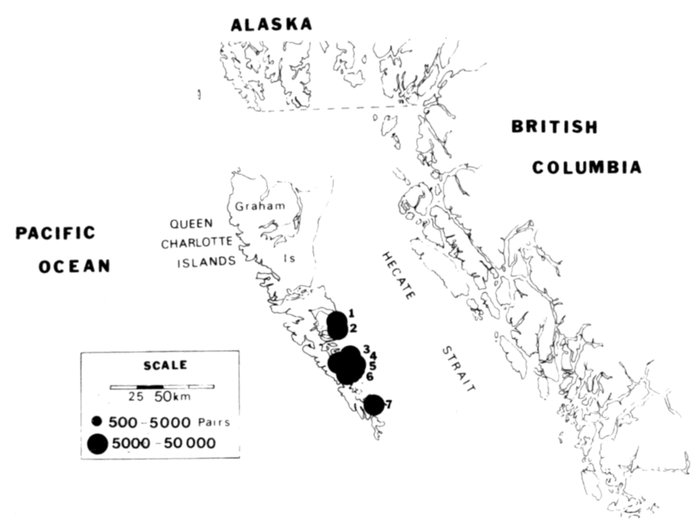
Fig. 2. Map of northern British Columbia showing sites of major seabird breeding colonies: 1—Skedans Island; 2—Limestone Island; 3—Agglomerate Island; 4—Bischoff Island; 5—Ramsey Island; 6—Alder Island; 7—Rankins Island.
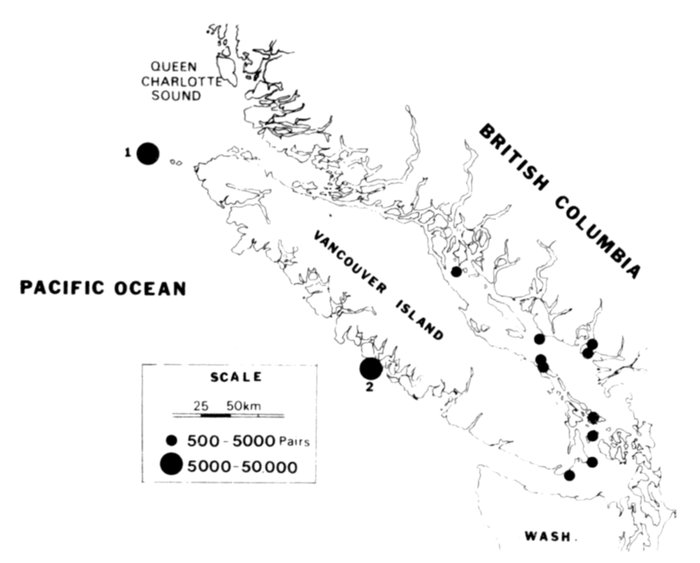
Fig. 3. Map of southern British Columbia showing sites of major seabird breeding colonies: 1—Triangle Island; 2—Cleland Island.
More than half of the breeding seabirds in British Columbia are found on the east coast of the Queen Charlotte Islands, and the fork-tailed storm-petrel (Oceanodroma furcata) comprises more than half of that total. However, new unpublished data (K. Vermeer) for Triangle Island and the northwest coast of Vancouver Island indicate that the population figures in Table 3 for this area are underestimates. Nevertheless, these two regions have nearly 80% of all the breeding seabirds in the Province. This results from the very large populations of the rhinoceros auklet and tufted puffin on Triangle Island and the fork-tailed storm-petrel, ancient murrelet, and Cassin's auklet on various islands on the east coast of the Queen Charlotte Islands (Table 3).
Continuing surveys of breeding seabirds are being conducted by personnel of the British Columbia Provincial Museum and the Canadian Wildlife Service.
Washington State
General Environment
For this report, we have distinguished two major geographical areas in Washington where breeding seabirds are found—the western coast of the Olympic Peninsula and the San Juan Islands, including the Strait of Juan de Fuca.
On the Olympic Peninsula, seabirds breed on the offshore rocks, islands, and precipitous cliffs from Copalis Beach to Cape Flattery (Fig. 4). The offshore rocks and islands throughout this area (except Tatoosh Island) are now included in the Washington Islands National Wildlife Refuge. Most of the larger rocks and islands have dense stands of salmonberry, salal, and grasses, and a few support stands of stunted conifers (Fig. 5); most are inaccessible to man. The adjacent coast is dominated by the Olympic rain forest where the mean annual precipitation is about 337.1 cm (U.S. Weather Bureau 1956, 1965a, 1965b).
Because the San Juan Islands lie northeast of the Olympic Peninsula and east of Vancouver Island (Fig. 6) they are in a rain shadow; however, because of highly variable topography and aspect, most islands have a diverse assemblage of plant communities (Franklin and Dyrness 1973). Exposed south-facing slopes are occupied by grassland vegetation and frequently by scattered trees, usually Pseudotsuga menziesii and Arbutus menziesii. Most of the seabird colonies are located on rather small exposed islands with short, grassy, shrubby vegetation. In general, these islands are not suitable for burrowing species.
Table 3.
Species composition, population estimates, and distribution of seabirds in British Columbia.
(+ = Present.)
Bird species Straits of Georgia and Juan de Fuca Southwest coast of Vancouver Island Northwest coast of Vancouver Island West coast of Queen Charlotte Island East coast of Queen Charlotte Island Prince Rupert to Queen Charlotte Island Total birds Percent of total
Fork-tailed storm-petrel + + 1,050 97,100 + 98,160 31.3
Leach's storm-petrel 10,000 + 1,800 180 750 12,730 4.1
Double-crested cormorant 1,058 0 0 0 0 0 2,116 >1.0
Brandt's cormorant 370 0 0 0 0 370 >1.0
Pelagic cormorant 2,174 336 3,350 1,456 496 12 9,998 3.2
Glaucous-winged gull 10,123 6,870 600 412 866 540 29,534 9.4
Common murre 16 3,000 0 0 0 3,016 1.0
Pigeon guillemot 1,029 204 250 358 1,458 1,650 5,978 1.9
Ancient murrelet 0 0 200 42,150 4 42,354 13.5
Cassin's auklet + 50,000 + 26,500 450 76,950 4.6
Rhinoceros auklet 1,200 + 10,000 300 200 11,700 3.7
Tufted puffin 1 154 20,000 190 0 42 20,388 6.5
Total 14,385 19,150 77,200 15,466 169,050 3,648 313,294 81.2
Table 4.
Breeding seabird population estimates for British Columbia
Geographic location Population estimate Percent of total
Straits of Georgia and Juan de Fuca 14,385 9.2
Southwest Coast of Vancouver Island 9,575 6.1
Northwest Coast of Vancouver Island 38,600 24.6
West Coast of Queen Charlotte Island 7,733 4.9
East Coast of Queen Charlotte Island 84,530 54.0
Prince Rupert to Queen Charlotte Strait 1,824 1.2
Total 156,647 100.0
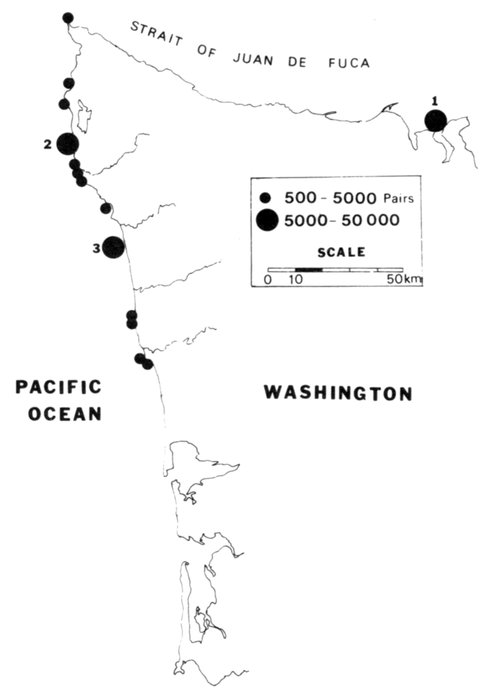
Fig. 4. Map of the Olympic Peninsula of Washington State showing sites of major seabird breeding colonies: 1—Protection Island; 2—Carroll Island; 3—Destruction Island.
In the Strait of Juan de Fuca, the two most important sites are Smith and Protection islands. Both are composed of glacial deposits and heavy sod that has developed under dense grassy vegetation (Fig. 7). Consequently, these two islands support most of the burrowing seabirds in the region. Unfortunately, both islands have historically been subjected to much human disturbance (Richardson 1961; Manuwal 1974).
The existing information on seabird colonies in both the coastal and San Juan Island areas has been largely derived from aerial surveys by the U.S. Fish and Wildlife Service. These surveys are inherently biased toward surface-nesting species such as gulls and cormorants. Population estimates for guillemots, auklets, storm-petrels, and puffins are less accurate. Some additional information obtained by direct island visitation has been provided by Kenyon and Scheffer (1961), Richardson (1961), Thoresen and Galusha (1971), G. Eddy (unpublished data), and D. A. Manuwal (unpublished data). Although other accounts of Washington seabirds are available, the references listed above are specifically oriented toward population assessment.
Olympic Peninsula
Despite the large number of offshore rocks, islets, and islands along the Pacific coast of Washington, significant seabird colonies are present only on about 30 islands. Since Table 5 summarizes the population estimates for 12 species of seabirds breeding on 24 major sites, it represents only the majority and not the total number of breeding seabirds on the Pacific coast of Washington. About 74% of the entire Washington seabird population resides on the coastal rocks and islands.
Major colony sites with more than 2,500 breeding pairs are Grenville Arch, Willoughby Rock, Destruction Island, Cake Rock, Carroll Island, and Bodelteh Island. More intensive censusing, especially of nocturnal burrowing species will undoubtedly raise the population estimates for these and other islands off the coast. About 54% of the total coastal population is composed of the common murre and rhinoceros auklet.
Fig. 5. Photograph of Destruction Island off the coast of Washington.
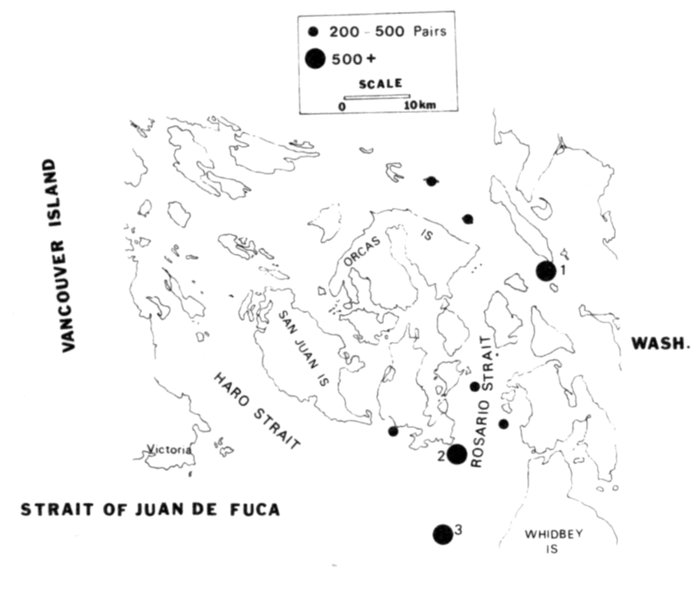
Fig. 6. Map of the San Juan Archipelago showing sites of major seabird breeding colonies: 1—Viti Rocks; 2—Colville Island; 3—Smith Island.
San Juan Islands
There are about 86 actual or potential seabird colony sites in this area; 25 (30%) are now considered important. Eleven islands are under Federal protection as National Wildlife Refuges. Part of Protection Island is owned by the Washington State Game Department to protect the largest rhinoceros auklet colony in the State. Most colony sites are on small islands with poorly developed soil which prevents burrowing species from using them. Consequently, the dominant species are surface nesters (such as gulls and cormorants) and rock-crevice nesters (like the pigeon guillemot). In all, about 31,000 seabirds of 7 species breed in the San Juan Island area. Breeding seabird population estimates for 49 of the 86 nesting sites are given in Table 6. Even though this does not represent all the colonies, it covers the most important islands and those islands where there appears to be potential for seabird breeding.
Fig. 7. Photograph of Smith Island in the Strait of Juan de Fuca, Washington. The glacial deposits are evident from the composition of the cliff faces.
Table 5.
Estimated breeding seabird populations of the outer coast of Washington
.
(Unpublished data from U.S. Fish and Wildlife Service and University of Washington)
Breeding site Species
Storm-petrels Cormorants Black oyster-catcher Gulls Common murre Pigeon guillemot Auklets Tufted puffin Total
Fork-tailed Leach's Unidentified Double-crested Brandt's Pelagic Western Glaucous-winged western Cassin's Rhinoceros
Copalis Rock — — 15 — — — — 30 — — — — — — 45
Point Grenville — — — 60 30 80 — 165 40 1,100 — — — — 1,475
Grenville Arch — — — 30 20 — 1 60 — 3,000 4 — — 3 3,118
Flat Rock — — 30 — — — — — 60 300 — — — — 390
Split Rock — — — 100 — — 1 150 — 2,100 4 — — — 2,355
Willoughby Rock — — — 80 40 15 — 150 — 3,000 — — — 25 3,310
South Rock — — — — — 40 — — 50 — — — — — 90
Abbey Islet — — — — — 30 3 — 50 — — — — 10 93
Destruction Island — — — — — — 12 350 — — 25 — 10,940 350 11,677
Middle Rock — — — — — 25 — — 25 — 50 — — — 100
North Rock — — — — — — — — 25 — — — — — 25
Alexander Island — — — — — 50 5 — 225 — — — — 1,550 1,830
Rounded Island — — — — — 25 — 25 — — 1 — — — 51
Giant's Graveyard — — — — — 10 — — — 150 — 50 150 — 360
Quillayute Needles — — — 50 50 50 — — 150 900 — — — 350 1,550
James Island — 30 — — — 40 — — 150 750 40 — — 20 1,030
Cake Rock — 500 — — — 150 — — 600 300 12 — 50 1,000 2,612
Sealion Rock — — — 70 — 30 — — 250 — — — — 5 355
Carroll Island — 3,100 — — — 100 3 — 550 — — 25 250 2,400 6,428
Ball Rock — — — — — 50 7 — 150 — — — — 750 957
White Rock — — — — — 100 — — 75 250 — — — 100 525
Ozette Island — — — — — — 1 — 15 — — — — — 16
Bodelteh Island 1,900 — — — — 100 2 — 300 — 5 — — 750 3,057
Tatoosh Island — 25 — — — 100 — — 1,500+ 100 20 25? 25? 30 1,825
Total 1,900 3,655 45 390 140 995 35 930 4,215 11,950 161 100 11,415 7,343 43,274
Table 6.
Breeding seabird population estimates for the San Juan Islands and Strait of Juan de Fuca, Washington, 1973-75
.
Breeding site Species
Cormorants Black oyster-catcher Glaucous-winged gull Pigeon guillemot Tufted puffin Rhinoceros Auklet Total
Double-crested Pelagic
Bare Island — 50 1 120 + — 2 173
Barren Island — — — — — — — 0
Battleship Island — — — — — — — 0
Bird Rocks 30 — + 320 — — — 350
Cactus Island — — 1 — — — — 1
Castle Island — — — — 30 — — 30
Colville Island — 40 1 1,000 — — — 1,041
Danger Island — — — 125 7 — — 132
Decatur Island — — — — — — — 0
Eliza Island — — — 3 1 — — 4
Eliza Rock — — — 1 — — — 1
Flat Top Island — — — — + — — +
Flower Island — 17 — 90 — — — 107
Goose Island — — — 60 — — — 60
Gull Rock — — + 125 7 — — 132
Gull Reef — — — — — — — 0
Hall Island — — 1 275 — — — 276
Harbor Rock — — — — — — — 0
Iceberg Island — — — — — — — 0
Johns Island — — 1 — — — — 1
Long Island — — 8 80 — — — 88
Low Island — — 1 75 17 — — 93
Lummi Rocks — — — 4 — — — 4
Matia Island — — — — + — — +
Mummy Rocks — — — 55 — — — 55
Minor Island — — — 100 — — — 100
O'Neal Island — — — — — — — 0
Patos Island — — — 20 + — — 20
North Peapod Island — — 1 220 2 — — 223
South Peapod Island — — 1 75 2 — — 78
Pearl Island — — — — — — — 0
Pointer Island — — — 58 2 — — 60
Protection Island 3 110 3 1,500 30 9,200 35 10,881
Puffin Island — — 1 350 15 — — 366
Ripple Island — — — — — — — 0
Sentinel Island — — — — 10 — — 10
Sentinel Rock — — 1 — — — — 1
Skip Jack Island — — — 75 20 — — 95
Smith Island — 20 6 10 30 600 — 666
Speiden Island — — — — — — — 0
South Sister Island 2 11 1 131 — — — 145
Middle Sister Island — — 1 22 — — — 23
North Sister Island — — 2 412 3 — — 417
Viti Rocks 29 80 1 387 1 — — 498
Waldron Island — — — — 2 — — 2
Williamson Rocks — 67 1 346 2 — — 416
Whale Island — — 1 70 — — — 71
White Rock — — + 125 13 — — 138
Yellow Island — — — — — — — 0
Total per species 64 395 34 6,234 194 9,800 37 16,758
Percent of total population 0.4 2.3 0.2 37.2 1.2 58.5 0.2 100.0
The major colony sites with more than 250 breeding pairs are located at Protection and Smith islands, Bird Rocks, Colville Island, Hall Island, North and South Peapod rocks, Puffin Island, North Sisters, Viti Rocks, and Williamson Rocks (Fig. 6). Glaucous-winged gulls are the predominant species on all these islands except Protection and Smith islands, where there are large colonies of rhinoceros auklets. Rhinoceros auklets (65%) and glaucous-winged gulls (32%) make up 97% of the total San Juan Islands seabird population.
Nest-site Preferences
Food supply and availability of nest sites are two critically important factors influencing the distribution and abundance of seabirds. Whereas information on general diet composition is known for most seabird species, we know little about the availability of favored seabird prey. The dynamics of seabird food chains is reviewed elsewhere in these proceedings.
The nest-site preferences for seabirds of the northeast Pacific Ocean are given in Table 7, and Table 8 indicates the proportion of seabirds that belong to specific nest-site categories. These preferences, in conjunction with knowledge of the physical characteristics of seabird habitat, permit a partial explanation of the present distribution and abundance of seabirds. For example, if we compare the San Juan Island habitats with those of the Washington coast, it is apparent that there are more cliff-nesting species on the coast. This reflects the physical characteristics of the two habitats. There are few cliffs in the San Juan Islands, and those that exist are very unstable. Colony sites in the San Juan Islands are typically on low, flat islands. Glaucous-winged gulls are the most abundant nesting species there. Coastal islands, on the other hand, are either covered by dense vegetation or are large monolithic chunks of rock with few available flat areas. Population estimates for the Washington coast are heavily biased toward surface nesters, since most of the data have been gathered by aerial surveys. Consequently, the burrow and rock crevice categories are underestimated. The aerial survey is appropriate for only about 43% of the birds nesting on the Washington coast.
Table 7.
Nest-site preference for seabirds breeding from Cape Fairweather, Alaska, to the Columbia River, Washington.
Nest-site type Bird species
Burrow-rock crevice
Diurnal Pigeon guillemot
Horned puffin
Tufted puffin
Nocturnal Fork-tailed storm-petrel
Leach's storm-petrel
Kittlitz's murrelet
Ancient murrelet
Cassin's auklet
Rhinoceros auklet
Open nests
Flat or slope Double-crested cormorant
Brandt's cormorant
Glaucous-winged gull
Herring gull
Western gull
Black oystercatcher
Cliff face Pelagic cormorant
Common murre
Black-legged kittiwake
Tree branch Marbled murrelet
Northern and southern British Columbia provide another good example of habitat availability as revealed through seabird population estimates. The population data are more comprehensive and have largely been gathered by island visitations. The islands in the northern portion are heavily vegetated and many have well-developed soil into which storm-petrels, auklets, and murrelets can burrow. Indeed, 96% of the seabird population consists of nocturnal, burrow-nesting species. In southern British Columbia, however, there are more open-nest species, particularly glaucous-winged gulls and cormorants.
Overall, 68% of the breeding seabirds found along the northeastern Pacific coast are nocturnal and nest in burrows or rock crevices (Table 8). The most conspicuous nesting birds such as gulls, cormorants, and murres, comprise only 22% of the total population. Consequently, our current estimates of breeding seabirds still underestimate the more secretive, nocturnal, burrow-nesting species.
Table 8.
Proportional nest-site preferences of Pacific coast seabirds.
Site Estimated number of pairs Percent of population Total
British Columbia San Juan Islands Washington coast British Columbia San Juan Islands Washington coast
Northern Southern Northern Southern Population Percent
Burrow-rock crevice
Diurnal 1,849 11,334 231 7,504 2.0 18.1 1.4 17.3 20,918 9.7
Nocturnal 90,347 30,600 9,800 17,070 96.0 48.9 58.6 39.4 147,817 68.1
Open nests
Flat or slope 909 15,101 6,298 5,755 1.0 24.2 37.6 13.3 28,063 13.0
Cliff face 982 5,525 395 12,945 1.0 8.8 2.4 30.0 19,847 9.2
Total 94,087 62,560 16,724 43,274 216,645
Population Changes
The available data are inadequate to detect changes in population distribution and density for most species (Table 9). In Washington, for instance, limited unsubstantiated information suggests an overall decline of the double-crested cormorant and tufted puffin in the San Juan Island area. Likewise, there seems to be an increase in glaucous-winged gulls there. In British Columbia, Drent and Guiguet (1961) were able to detect changes in some species. For example, they noted increases in the double-crested cormorant, pelagic cormorant, and glaucous-winged gull. No change was observed in the tufted puffin. Since then, the Brandt's cormorant has established a colony in Barkley Sound (Guiguet 1971). The data in southeastern Alaska are inadequate for all species except, perhaps, the Cassin's auklet which Gabrielson and Lincoln (1959) reported to be declining throughout Alaska. In short, no definitive statements can now be made concerning changes in seabird population numbers.
Species Accounts
Fork-tailed Storm-petrel (Oceanodroma furcata)
Storm-petrels are especially difficult to census because they are nocturnal, and the burrows and rock crevices where they breed are often difficult to locate, especially in mixed-species colonies. The census data are inadequate to determine whether there have been changes in population density and distribution. Indeed, the biology of this species is perhaps the least known of the North Pacific colonial seabirds. In southeastern Alaska, this species is outnumbered by at least 5 to 1 by the Leach's storm-petrel (Oceanodroma leucorhoa). The reasons for this are poorly understood. There is some evidence that the numbers of breeding fork-tailed storm-petrels on Forrester Island may fluctuate drastically from one year to the next (Gabrielson and Lincoln 1959).
Leach's Storm-petrel (Oceanodroma leucorhoa)
Of the two subspecies of this petrel (O. l. leucorhoa and O. l. beali), only O. l. beali is found in southeastern Alaska. The leucorhoa subspecies is more northerly in distribution. Where both fork-tailed and Leach's storm-petrels are sympatric, Leach's predominates; however, this relationship becomes more unpredictable in British Columbia and Washington. This species is undoubtedly widespread in the forested islands of the Alexander Archipelago.
Double-crested Cormorant (Phalacrocorax auritus)
The double-crested cormorant apparently does not breed in southeastern Alaska since Willett (1912), Gabrielson and Lincoln (1959), and S. Patten (personal communication) do not report breeding colonies for the area. The largest populations occur in southern British Columbia principally in the Gulf Islands, where 71% of all breeding double-crested cormorants are found (Table 10). According to Jewett et al. (1953), this species was less common in Puget Sound than was Brandt's cormorant, but is certainly not the case today (D. A. Manuwal, unpublished data). The only common cormorants in the San Juan Islands are the pelagic and double-crested species. The double-crested cormorant seems to have declined in numbers on both coastal and inland waters. On the basis of his observations, R. W. Campbell believes that this species is increasing in British Columbia.
Table 9.
Distribution and status of marine birds breeding along the Pacific coast of Washington, British Columbia, and southeastern Alaska.
(X = known to breed in the region;? = data insufficient; + = evidence indicates an overall increase in size of population; - = evidence indicates an overall decrease in size of population; 0 = no population change.)
Family and species Common name Washington British Columbia Southeastern Alaska
Presence Status Presence Status Presence Status
Hydrobatidae
Oceanodroma furcata Fork-tailed storm-petrel X ? X ? X ?
O. leucorhoa Leach's storm-petrel X ? X - X ?
Phalacrocoracidae
Phalacrocorax auritus Double-crested cormorant X - X -
P. penicillatus Brandt's cormorant X ? X 0 ?
P. pelagicus Pelagic cormorant X ? X + X ?
Haematopodidae
Haematopus bachmani Black oystercatcher X ? X + X ?
Laridae
Larus glaucescens Glaucous-winged gull X + X + X ?
L. occidentalis Western gull X ? X ?
L. argentatus Herring gull X ?
Rissa tridactyla Black-legged kittiwake X ?
Alcidae
Uria aalge Common murre X ? X - X ?
Cepphus columba Pigeon guillemot X ? X + X ?
Brachyramphus marmoratus Marbled murrelet X ? X ? X ?
B. brevirostris Kittlitz's murrelet X ?
Synthliboramphus antiquus Ancient murrelet X ? X ?
Ptychoramphus aleuticus Cassin's auklet X ? X ? X -
Cerorhinca monocerata Rhinoceros auklet X ? X + X ?
Fratercula corniculata Horned puffin X ?
Lunda cirrhata Tufted puffin X - X 0 X ?
Total species 14 15 16
Brandt's Cormorant (Phalacrocorax penicillatus)
Brandt's cormorant is the least abundant of the three cormorant species that nest in the study area. Washington is at the northernmost edge of the breeding distribution of this species. Only one more northerly colony exists, on Sartine Island off Vancouver Island (Vermeer et al. 1976). Brandt's cormorant comprises about 85% of the cormorant population in Oregon (U.S. Fish and Wildlife Service, unpublished data). However, in Washington it is only about 9% and in British Columbia 3% of the total cormorant population.
Table 10.
Estimated seabird populations breeding from Cape Fairweather, Alaska, to the Columbia River, Washington.
(? = present in unknown numbers; - = inadequate data.)
Bird species Northern British Columbia Southern British Columbia San Juan Islands Washington coast Total all regions
Population Percent Population Percent Population Percent Population Percent Population Percent
Fork-tailed storm-petrel 49,080 52.2 ? - 0 - 1,900 4.4 50,980 23.5
Leach's storm-petrel 1,365 1.5 5,000 8.0 0 - 3,655 8.5 10,020 4.6
Double-crested cormorant 0 - 1,058 1.7 64 >0.1 390 >0.1 1,512 >0.1
Brandt's cormorant 0 - 185 >0.1 0 - 140 >0.1 325 >0.1
Pelagic cormorant 982 1.0 4,017 6.4 395 2.4 995 2.3 6,389 3.0
Glaucous-winged gull 909 1.0 13,858 22.2 6,234 37.3 4,215 9.8 25,216 11.6
Western gull 0 - ? - 0 - 930 2.2 930 >0.1
Common murre 0 - 1,508 2.4 0 - 11,950 27.7 13,458 6.2
Pigeon guillemot 1,733 1.8 1,256 2.0 194 1.2 161 >0.1 3,345 1.5
Ancient murrelet 21,177 22.5 0 - 0 - 0 - 21,177 9.8
Cassin's auklet 13,475 14.3 25,000 40.0 0 - 100 >0.1 38,575 17.8
Rhinoceros auklet 5,250 5.6 6,000 >0.1 9,800 58.6 11,415 26.4 27,065 12.5