PART I. RESPONSE OF PLANT ORGANS. (continued 2)
Reading edition
7. The action of chemical agents.
8. Effect of “fatigue” on response.
9. The influence of constant electric current on recovery.
10. The action of light and darkness on excitability.
The isolated petiole-pulvinus preparation is made by cutting out a portion of the stem bearing a single lateral leaf. The four diverging sub-petioles may also be cut off. In order to prevent rapid drying the specimen has to be kept in water. Preparations made in this way often appeared to have lost their sensibility. I was, however, able to trace this loss to two different factors: first, to the physiological depression due to injury caused by section, and, second, to the sudden increase of turgor brought on by excessive absorption of water. I shall now proceed to show that the loss of sensibility is not permanent, but is capable of restoration.
EFFECT OF WOUND OR SECTION IN MODIFICATION OF NORMAL EXCITABILITY.
In connection with the question of effect of injury, it is to be borne in mind that after each excitation the plant becomes temporarily irresponsive and that the excitability is fully restored after the completion of protoplasmic recovery. A cut or a section acts as a very intense stimulus, from the effect of which the recovery is very slow. If the stem be cut very near the leaf, the excitation of the pulvinus is very intense, and the consequent loss of excitability becomes more or less persistent. But if the stem be cut at a greater distance, the transmitted excitation is less intense, and the cut specimen recovers its excitability within a moderate time. I have also succeeded in reducing the excitatory depression by previously benumbing the tissue by physiological means. The isolated specimen can be made still more compact by cutting off the sub-petioles bearing the leaflets; the preparation now consists of a short length of stem of about 2 cm. and an equally short length of primary petiole, the motile pulvinus being at the junction of the two.
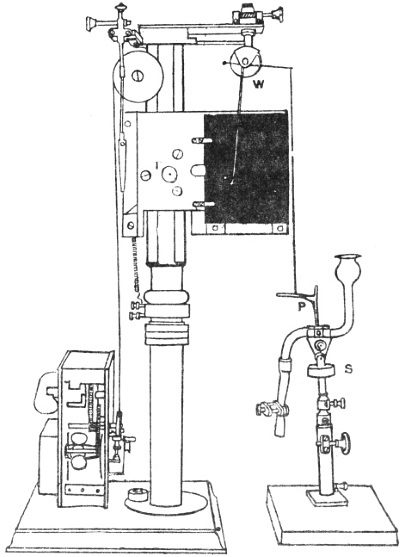
Fig. 30—The Resonant Recorder, with petiole-pulvinus preparation. (From a photograph.)
For the restoration of sensitiveness, and to meet working conditions, the lower end of the cut stem is mounted on a T-tube, with funnel-attachment and exit-tube, as shown in Fig. 30. The other two cut ends—of the stem and of the petiole—may be covered with moist cloth or may be closed with collodion flexile to prevent rapid evaporation and drying up of the specimen. A slight hydrostatic pressure maintains the specimen in a moderately turgid condition. A preparation thus made is insensitive at the beginning, but if left undisturbed it slowly recovers its excitability. The history of the depression of excitability after shock of preparation and its gradual restoration is graphically illustrated by a series of records made by the plant (Fig. 31).
The petiole-pulvinus preparation thus made offers all facilities for experiment. Owing to its small size it can be easily manipulated; it can be enclosed in a small chamber and subjected to varying conditions of temperature and to the action of different vapours and gases. Drugs are easily absorbed at the cut end, and poison and its antidote can be successively applied through the funnel without any disturbance of the continuity of record. In fact, many experiments which would be impossible with the entire plant are quite practicable with the isolated leaf.
The arrangement for taking records of response is seen in Fig. 30, which is reproduced from a photograph of the actual apparatus. For recording the response and recovery of the leaf under stimulation, I use my Resonant Recorder fully described in the ‘Philosophical Transactions’ (1913). The petiole is attached to one arm of the horizontal lever. The writer, made of fine steel wire with a bent tip, is at right angles to the lever, and is maintained by electromagnetic means in a state of to-and-fro vibration, say, ten times in a second. The record, consisting of a series of dots, is free from errors arising from friction of continuous contact of the writer with the recording surface. The successive dots in the record at definite intervals of a tenth of a second also give the time-relations of the response curve.
On account of its small size, the petiole-pulvinus preparation offers great facilities for mounting in different ways suitable for special investigations. Ordinarily, the cut stem with its lower end enclosed in moist cloth is supported below. A very suitable form of stimulus is that of induction shock from a secondary coil, the intensity of which is capable of variation in the usual manner by adjusting the distance between the primary and the secondary coils. The motile pulvinus, P, may be excited directly. For investigations on velocity of transmission of excitation, stimulus is applied on the petiole at some distance from the pulvinus, by means of suitable electrodes. Excitation is now transmitted along the intervening length of petiole, the conducting power of which will be found appropriately modified under the action of chemical and other agents. In this normal method of mounting, the more excitable lower half of the pulvinus is below; excitatory reaction produces the fall of the petiole, gravity helping the movement. The preparation may, however, be mounted in the inverted position, with the more excitable lower half of the pulvinus facing upwards. The excitatory movement will now be the erection of the petiole, against gravity.
Under natural conditions the stem is fixed, and it is the petiole which moves under excitation. But a very interesting case presents itself when the petiole is fixed and the stem free. Here is presented the unusual spectacle of the plant or the stem “wagging” in response to excitation.
THE CHANGE OF EXCITABILITY AFTER IMMERSION IN WATER.
The isolated specimen can be kept alive for several days immersed in water. The excitability of the pulvinus, however, undergoes great depression, or even abolition, by the sudden change of turgor brought on by excessive absorption of water. The plant gradually accommodates itself to the changed condition, and the excitability is restored in a staircase manner from zero to a maximum.
In studying the action of a chemical solution on excitability, the solution may be applied through the cut end or directly on the pulvinus. The sudden variation of turgor, due to the liquid, always induces a depression, irrespective of the stimulating or the depressing action of the drug. The difficulty may be eliminated by previous long-continued application of water on the pulvinus and waiting till the attainment of uniform excitability which generally takes place in the course of about three hours. Subsequent application of a chemical solution gives rise to characteristic variation in the response.
QUANTITATIVE DETERMINATION OF THE RATE OF DECAY OF EXCITABILITY IN AN ISOLATED PREPARATION.
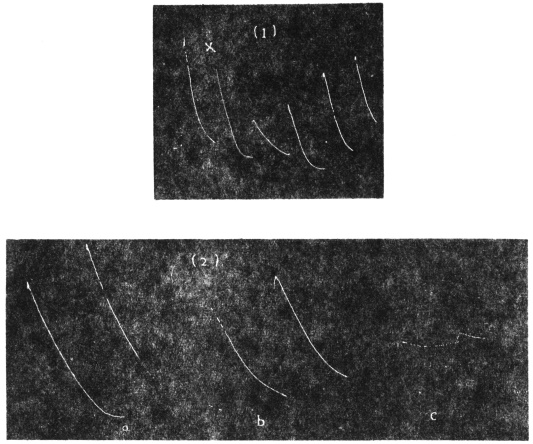
Fig. 31—Variation of excitability after section. (1) Immediate effect; (2) variation of excitability in a second specimen during 50 hours: (a) response 4 hours after section; (b) response after 24 hours; (c) after 49 hours. Up-line of record represents responsive fall of the leaf, down-line indicates recovery from excitation.
Variation of excitability after section: Experiment 23.—In order to test the history of the change of excitability resulting from the immediate and after-effect of section, I took an intact plant and fixed the upper half of the stem in a clamp. The response of a given leaf was now taken to the stimulus of an induction shock of 0.1 unit intensity, the unit chosen being that which causes a bare perception of shock in a human being. The specimen was vigorous and the response obtained was found to be a maximum. The stem bearing the leaf was cut at the moment marked in the record with a cross, and water was applied at the cut end. The effect of section was to cause the maximum fall of the leaf, with subsequent recovery. After this, successive responses to uniform stimuli at intervals of 15 minutes show, in (1) of Fig. 31, that a depression of excitability has been induced owing to the shock caused by section. In course of an hour, however, the excitability had been restored almost to its original value before the section. This was the case with a vigorous specimen, but with less vigorous ones a longer period of about three hours is required for restoration. In certain other cases the response after section exhibits alternate fatigue; that is to say, one response is large and the next feeble, and this alternation goes on for a length of time. The isolated specimen, generally speaking, attains a uniform sensibility after a few hours, which is maintained, with very slight decline under constant external conditions, for about 24 hours. On the third day the fall of excitability is very rapid, and the sensibility declines to zero in about 50 hours after isolation [Fig. 31 (2)]. We may describe the whole cycle of change as follows: by the shock of operation the isolated preparation is rendered insensitive for nearly an hour, the excitability is then gradually restored almost to its normal value before operation. Under constant external conditions, this excitability remains fairly constant for about 24 hours after which depression sets in. The rate of fall of excitability becomes very rapid 40 hours after the operation, being finally abolished after the fiftieth hour. It is probable that in a colder climate the fall of excitability would be much slower. The most important outcome of this inquiry is the demonstration of the possibility of obtaining persistent and uniform sensibility in isolated preparations. On account of this, not only is the difficulty of supply of material entirely removed but a very high degree of accuracy secured for the investigation itself.
EFFECT OF AMPUTATION OF UPPER HALF OF PULVINUS.
Experiment 24.—The determination of the rôle played by different parts of the pulvinus in response and recovery is of much theoretical importance. Our knowledge on this subject is unfortunately very scanty. The generally accepted view is that on excitation “the actual downward curvature of the pulvinus is partly due to a contraction of the walls of the motor cells consequent upon the decrease of turgor, but is accentuated by expansion of the insensitive adaxial half of the pulvinus—which was strongly compressed in the unstimulated condition of the organ—and also by the weight of the leaf.”[H] According to Pfeffer, after excitation of the organ, “the original condition of turgor is gradually reproduced in the lower half of the pulvinus, which expands, raising the leaf and producing compression of the upper half of the pulvinus, which aids in the rapid curvature of the stimulated pulvinus.”[I]
It was held, then, that the rapidity of the fall of leaf under stimulus is materially aided (1) by the expansion of the upper half of the pulvinus, which is normally in a state of compression, and (2) by the weight of the leaf. So much for theory. The experimental evidence available regarding the relative importance of the upper and lower halves of the pulvinus is not very conclusive. Lindsay attempted to decide the question by his amputation experiments. He showed that when the upper half was removed the leaf carried out the response, but rigor set in when the lower half was amputated. Pfeffer’s experiments on the subject, however, contradicted the above results. He found that “after the upper half of the pulvinus was carefully removed, no movement was produced by stimulation, whereas when the lower half is absent a weakened power of movement is retained.” Pfeffer, however, adds, “since the operation undoubtedly affects the irritability, it is impossible to determine from such experiments the exact part played by the active contraction of the lower half of the pulvinus.”[I]
The cause of uncertainty in this investigation is twofold. First, it arises from the unknown change in irritability consequent on amputation; and, secondly, from absence of any quantitative standard by which the effect of selective amputation of the pulvinus may be measured. As regards the first, I have been able to reduce the depressing action caused by injury to a minimum by benumbing the tissue before operation, through local application of cold, and also allowing the shock-effect to disappear after a rest of several hours. As regards the physiological gauge of efficiency of the motor mechanism, such a measure is afforded by the relation between a definite testing stimulus and the resulting response with its time-relations, which is secured by my Resonant Recorder with the standardised electrical stimulator.
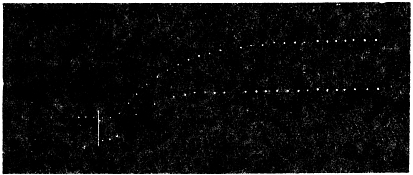
Fig. 32—Effect of amputation of upper half of pulvinus. Upper record gives normal response before amputation, and the lower, response after amputation. (Successive dots at intervals of 0.1 sec). Apex-time 11 sec, in both.
In carrying out this investigation I first took the record of normal response of an intact leaf on a fast moving plate. A second record, with the same stimulus, was taken after the removal of the upper half of the pulvinus, having taken the necessary precautions that have been described. Comparison of the two records (Fig. 32) shows that the only difference between them is in the exhibition of slight diminution of excitability due to operation. But, as regards the latent period and the quickness of attaining maximum fall, there is no difference between the two records before and after the amputation of the upper half. The upper part of the pulvinus is thus seen practically to have little influence in hastening the fall.
EFFECT OF REMOVAL OF THE LOWER HALF.
Experiment 25.—The shock-effect caused by the amputation of the lower half was found to be very great, and it required a long period of rest before the upper half regained its excitability. The excitatory reaction of the upper half is by contraction, and the response is, therefore, the lifting of the petiole. Thus, in an intact specimen, excitation causes antagonistic reactions of the two halves. But the sensibility of the upper half is very feeble and the rate of its contractile movement, relatively speaking, very slow. The record of the response of the upper half of the pulvinus, seen in Fig. 33, was taken with an Oscillating Recorder, where the successive dots are at intervals of 1 sec.: the magnification employed was about five times greater than in recording the response of the lower half (Fig. 32). The intensity of stimulus to evoke response had also to be considerably increased. Taking into account the factors of magnification and the intensity of stimulus for effective response, the lower half I find to be about 80 times more sensitive than the upper. Thus, under feeble stimulus the upper half exerts practically no antagonistic reaction. The excitatory response of the upper half is also seen to be very sluggish.
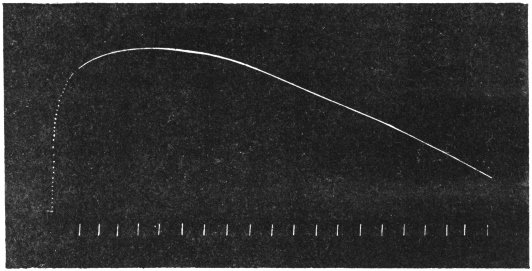
Fig. 33.—Response after amputation of lower half of pulvinus. (Successive dots at intervals of a second; vertical lines mark minutes.) Apex-time, 40 secs.
INFLUENCE OF THE WEIGHT OF LEAF ON RAPIDITY OF RESPONSIVE FALL.
Experiment 26.—It is obvious that the mechanical moment exerted by the weight of the leaf must help its responsive fall under excitation. But the relative importance of the factors of active contraction of the lower half of the pulvinus and of the weight, in the rate of the responsive down-movement, still remains to be determined. A satisfactory way of solving the problem would lie in the study of the characteristics of response-records taken under three different conditions: (1) When the leaf is helped in its fall by its weight; (2) when the action of the weight is eliminated; and (3) when the fall has to be executed against an equivalent weight. An approximation to these conditions was made in the following manner. We may regard the mechanical moment to be principally due to the weight of the four sub-petioles applied at the end of the main petiole. In a given case these sub-petioles were cut off, and their weight found to be 0.5 grm. The main petiole was now attached to the right arm of the lever, and three successive records were taken: (1) With no weight attached to the petiole; (2) with 0.5 grm. attached to its end; and (3) with 0.5 grm. attached to left arm of the lever at an equal distance from the fulcrum. In the first case, the fall due to the excitatory contraction will practically have little weight to help it; in the second case, it will be helped by a weight equivalent to those of the sub-petioles with their attached leaflets; and in the third case, the fall will be opposed by an equivalent weight. We find that in these three cases there is very little difference in the time taken by the leaf to complete the fall (Fig. 34).
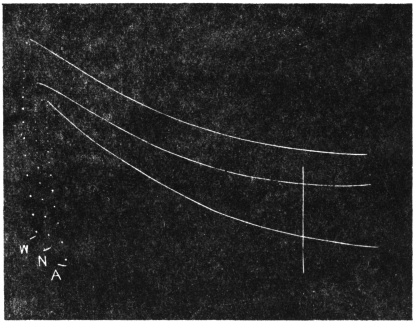
Fig. 34.—Effect of weight on rapidity of fall. N, without action of weight; W, with weight helping; and A, with weight opposing.
It has been shown that the presence or absence of the upper half of the pulvinus makes practically no difference in the period of fall; it is now seen that the weight exerts comparatively little effect. We are thus led to conclude that in determining the rapidity of fall, the factors of expansive force of the upper half of the pulvinus and the weight of the leaf are negligible compared to the active force of contraction exerted by the lower half of the pulvinus.
ACTION OF CHEMICAL AGENTS.
In connection with this subject it need hardly be said that the various experiments which I had previously carried out with the intact plant can also be repeated with the isolated preparation. I will only give here accounts of experiments which are entirely new.
The chemical solution may be applied directly to the pulvinus, or it may be absorbed through the cut end, the absorption being hastened by hydrostatic pressure. The normal record is taken after observing precautions which have already been mentioned. The reaction of a given chemical agent is demonstrated by the changed character of the record. The effect of the drug is found to depend not merely on its chemical nature, but also on the dose. There is another very important factor—that of the tonic condition of the tissue—which is found to modify the result. The influence of this will be realised from the account of an experiment to be given presently, where an identical agent is shown to produce diametrically opposite effects on two specimens, one of which was in a normal, and the other in a sub-tonic, condition. The experiments described below relate to reactions of specimens in a normal condition.
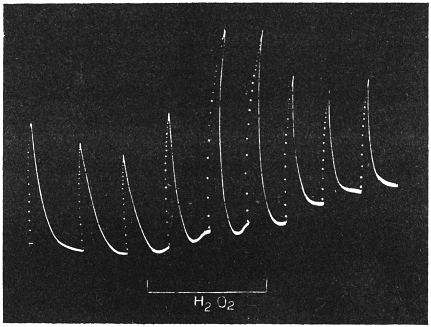
Fig. 35.—Stimulating action of hydrogen peroxide.
Hydrogen Peroxide: Experiment 27.—This reagent in dilute solution exerts a stimulating action. Normal records, were taken after long-continued application of water on the pulvinus. The peroxide, as supplied by Messrs. Parke Davis & Co., was diluted to 1 per cent., and applied to the pulvinus; this gave rise to an enhancement of response. Re-application of water reduced the amplitude to the old normal value (Fig. 35).
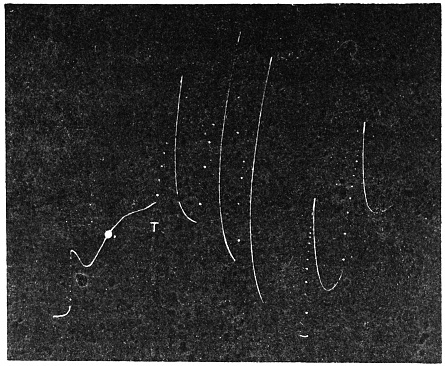
Fig. 36.—Incomplete recovery under the action BaCl2 and transient restoration under tetanisation at T.
Barium Chloride: Experiment 28.—The action of this agent is very characteristic, inducing great sluggishness in recovery. The preparation had been kept in 1-per cent. solution of this substance for two hours. After this the first response to a given test-stimulus was taken; the response was only moderate, and the recovery incomplete. The sluggishness was so great that the next stimulation, represented by a thick dot (Fig. 36), was ineffective. Tetanising electric shock at T, not only brought about response, but removed for the time being the induced sluggishness. This is seen in the next two records, which were taken under the old test-stimulus. There is now an enhanced response and a complete recovery. Beneficial effect of tetanisation disappeared, however, on the cessation of stimulus. This is seen in the next two records which were taken after two hours. The amplitude of response was not only diminished, but the recovery also was incomplete.
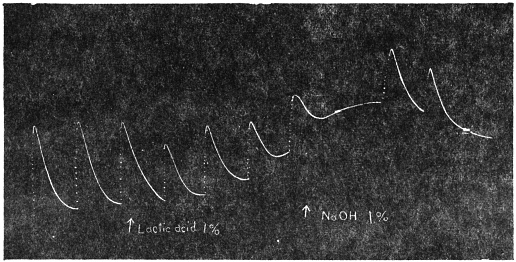
Fig. 37.—Antagonistic action of alkali and acid. Arrest of response in contraction under NaOH (↑), restoration and final arrest in expansion under lactic acid. (↑)
Antagonistic actions of Alkali and Acid: Experiment 29.—Alkali and acid are known to exert antagonistic actions on the spontaneous beat of the heart; dilute solution of NaOH arrests the beat of the heart in systolic contraction, while dilute lactic acid arrests the beat in diastolic expansion. I have found identical antagonistic reactions in the pulsating tissue of Desmodium gyrans, the telegraph plant. It is very interesting to find that these agents also exert their characteristic effects on the response of Mimosa in a manner which is precisely the same. This is seen illustrated in Fig. 37, where the application of NaOH arrested the response in a contracted state; after this, the antagonistic effect of dilute lactic acid is seen first, in its power of restoring the excitability; its continued application, however, causes a second arrest, but this time in a state of relaxed expansion.
CuSO4 Solution.—This agent acts as a poison, causing a gradual diminution of amplitude of response, culminating in actual arrest at death. Certain poisons, again, exhibit another striking symptom at the moment of death, an account of which will be given in a separate paper.
EFFECT OF “FATIGUE” ON RESPONSE.
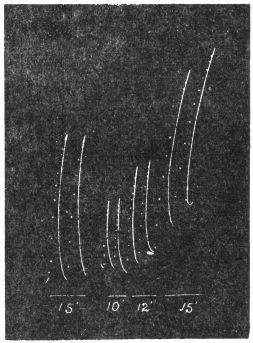
Fig. 38.—“Fatigue” induced by shortening intervening period of rest.
With Mimosa, after each excitation the recovery becomes complete after a resting period of about 15 min. With this interval of rest the successive responses for a given stimulus are equal, and are at their maximum.
Experiment 30.—When the resting interval is diminished the recovery becomes incomplete, and there is a consequent diminution of amplitude of response. There is thus an increased fatigue with diminished period of rest. This is illustrated in Fig. 38, where the first two responses are at intervals of 15 min.; the resting interval was then reduced to 10 min., the response undergoing a marked diminution. Conversely, by increasing the resting interval, first to 12 and then to 15 min., the extent of fatigue was reduced and then abolished.
THE INFLUENCE OF CONSTANT ELECTRIC CURRENT ON RECOVERY.
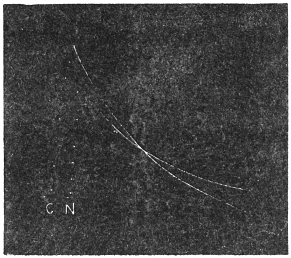
Fig. 39.—Action of constant current in removal of fatigue by hastening recovery; N, curve of response in fatigued specimen; C, after passage of current.
Experiment 31.—From the above experiment it would appear that since the incompleteness of recovery induces fatigue, hastening of recovery would remove it. With this idea I tried various methods for quickening the recovery of the excited leaf. The application of a constant electric current was found to have the desired effect. Two electrodes for introduction of current were applied, one on the stem and the other on the petiole, at some distance from the pulvinus. In order to avoid the excitatory effect of sudden application, the applied current should be increased gradually; this was secured by means of a potentiometer slide. In my experiment a current having an intensity of 1.4 micro-ampère was found to be effective. Responses at intervals of 10 min., as we have seen, exhibit marked fatigue. Two responses were recorded on a fast-moving plate, N before, and C after, the application of the current. It will be seen (Fig. 39) how the application of current has, by hastening the recovery, enhanced the amplitude of response and brought about a diminution of fatigue. In connection with this, I may state that the tonic condition is, in general, improved as an after-effect of the passage of current. This is seen in some cases by a slight increase in excitability; in others, where the responses had been irregular, the previous passage of a current tends to make the responses more uniform.
ACTION OF LIGHT AND DARKNESS ON EXCITABILITY.
In taking continuous records of responses I was struck by the marked change of excitability exhibited by the intact plant under variation of light. Thus the appearance of a cloud was quickly followed by an induced depression, and its disappearance by an equally quick restoration of excitability. This may be explained on the theory that certain explosive chemical compounds are built up by the photosynthetic processes in green leaves, and that the intensity of response depends on the presence of these compounds. But the building up of a chemical compound must necessarily be a slow process, and it is difficult on the above hypothesis to connect the rapid variation of excitability with the production of a chemical compound, or its cessation, concomitant with changes in the incident light.
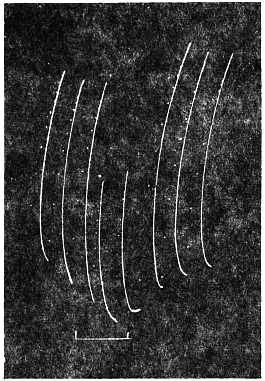
Fig. 40.—Stimulating action of light, and depressing action of darkness. Horizontal line below represents period of darkness.
Experiment 32.—In order to find out whether photo-synthesis had any effect on excitability, I placed an intact plant in a dark room and obtained from it a long series of responses under uniform test-stimulus. While this was being done the green leaflets were alternately subjected to strong light and to darkness, care being taken that the pulvinus was shaded all the time. The alternate action of light and darkness on leaflets induced no variation in the uniformity of response. This shows that the observed variation of excitability in Mimosa under the alternate action of light and darkness is not attributable to the photo-synthetic processes.
I next took a petiole-pulvinus preparation from which the sub-petioles bearing the leaflets had been cut off, and placed it in a room illuminated by diffused daylight. The normal responses were taken, the temperature of the room being 30°C. The room was darkened by pulling down the blinds, and records were continued in darkness. The temperature of the room remained unchanged at 30°C. It will be seen from records given in Fig. 40, that in darkness there is a great depression of excitability. Blinds were next pulled up and the records now obtained exhibit the normal excitability under light. The sky had by this time become brighter, and this accounts for the slight enhancement of excitability. This experiment proves conclusively that light has a direct stimulating action on the pulvinus, independent of photo-synthesis.[J]
SUMMARY.
On isolation of a petiole-pulvinus preparation, the shock of operation is found to paralyse its sensibility. After suitable mounting the excitability is restored, and remains practically uniform for nearly 24 hours. After this a depression sets in, the rate of fall of excitability becomes rapid 40 hours after the operation, sensibility being finally abolished after the fiftieth hour.
Experiments carried out on the effect of weight, and the influence of selective amputation of the upper and lower halves of the pulvinus, show that in determining the rapidity of fall of leaf, the assumed factors of the expansive force of the upper half of the pulvinus and the weight of the leaf are negligible compared to the force of active contraction exerted by the lower half of the pulvinus. The excitability of the lower half is eighty times greater than that of the upper.
Chemical agents induce characteristic changes in excitability. Hydrogen peroxide acts as a stimulant. Barium chloride renders the recovery incomplete: but tetanisation temporarily removes the induced sluggishness. Acids and alkalis induce antagonistic reactions, abolition of excitability with alkali taking place in a contracted, and with acid in an expanded condition of the pulvinus.
The responses exhibit fatigue when the period of rest is diminished. The passage of constant current is found to remove the fatigue.
Response is enhanced on exposure to light, and diminished in darkness. Light is shown to exert a direct stimulating action on the pulvinus, independent of photo-synthesis.
VI.—ON CONDUCTION OF EXCITATION IN PLANTS
By
Sir J. C. Bose.
The plant Mimosa offers the best material for investigation on conduction of excitation. With regard to this question the prevailing opinion had been that in plants like Mimosa, there is merely a transmission of hydro-mechanical disturbance and no transmission of true excitation comparable with the animal nerve. I have, however, been able to show that the transmission in the plant is not a mechanical phenomenon, but a propagation of excitatory protoplasmic change. This has been proved by the arrest of conduction by the application of various physiological blocks. Thus local application of increasing cold retards, and finally abolishes the conducting power. The conducting tissue becomes paralysed for a time as an after-effect of application of cold; the lost conducting power may, however, be quickly restored by tetanising electric shocks. The conducting power of an animal nerve is arrested by an electrotonic block, the conductivity being restored on the cessation of the current. I have succeeded in inducing similar electrotonic block of conduction in Mimosa. Conductivity of a selective portion of petiole may also be permanently abolished by local action, of poisonous solution of potassium cyanide.[K]
Having thus established the physiological character of the transmitted impulse in plants I shall now proceed to give some of the principal results of my earlier and recent investigations on the effects of various agencies on conduction of excitation in plants.
Apart from any question of hydro-mechanical transmission, it is important to distinguish two different modes of transmission of excitation. In a motile tissue contraction of a cell causes a physical deformation and stimulation of the neighbouring cell. Examples of this are furnished by the cardiac muscle of the animal, the pulvinus of Mimosa, and the stamen of Berberis. This mode of propagation may better be described as a convection of excitation.
The conduction of excitation, as in a nerve, is a different process of transmission of protoplasmic change. The conducting tissue in this case does not itself exhibit any visible change of form. In the plant the necessary condition for transmission of excitation to a distance is that the conducting tissue should be possessed of protoplasmic continuity in a greater or less degree. This condition is fulfilled by vascular bundles. There being greater facility of transmission along the bundles than across them, the velocity in the longitudinal direction is very much greater than in the transverse.
For accurate determination of velocity of transmission the testing stimulus should be quantitative and capable of repetition. Abnormal high velocity has been observed in Mimosa by applying crude and drastic methods of stimulation, by a transverse cut or a burn. This is apt to give rise to a very strong hydro-dynamic disturbance, which travelling with great speed, delivers a mechanical blow on the responding pulvinus. Such hydro-dynamic transmission is not the same as physiological conduction.
In the primary petiole of Mimosa the highest velocity under electric stimulation I find to be about 30 mm. per second. This velocity is considerably lower than the velocity in the nerve of higher animals, but higher than in the lower animals. As an example of the latter, mention may be made of the velocity of 10 mm. per second in the nerve of Anodon and 1 mm. per second in the nerve of Eledone.
PREFERENTIAL DIRECTION OF CONDUCTION.
Experiment 33.—The conduction of excitatory impulse takes place in both directions. This can be demonstrated by taking a petiole of Biophytum sensitivum or of Averrhoa carambola. These petioles are provided with a series of motile leaflets. Stimulation at the middle point of the petiole gives rise to two waves of excitation, one of which travels towards the central axis of the plant, and the other away from it. The centrifugal velocity is greater than the centripetal as will be seen from the following results:
BiophytumVelocity in centrifugal direction2.90 mm per second.
" centripetal " 2.00 mm " "
Averrhoa " centrifugal " 0.50 mm " "
" centripetal " 0.26 mm " "
EFFECT OF TEMPERATURE.
Variation of temperature has a marked effect on the velocity of transmission of excitation. Lowering of temperature diminishes the velocity, culminating in an arrest. Rise of temperature, on the other hand, enhances the velocity. This enhancement is considerable in specimens in which the normal velocity is low, but in plants in optimum condition, the velocity being already high, cannot be further enhanced. The following tabular statement gives results of effects of temperature on velocity of transmission in Mimosa and Biophytum:—
TABLE IV.—EFFECT OF TEMPERATURE ON VELOCITY OF TRANSMISSION.
Specimen.Temperature.Velocity.
Mimosa (winter specimen)22°C3.6 mm. per second.
28°C6.3 mm. " "
31°C9.0 mm. " "
Biophytum30°C3.7 mm. " "
35°C7.4 mm. " "
37°C9.1 mm. " "
EFFECT OF SEASON.
The velocity of transmission is very much lower in winter than in summer. In the petiole of Mimosa, the velocity in summer is as high as 30 mm. per second; in winter it is reduced to about 4 mm. The lowering of velocity in winter is partly due to the prevailing low temperature and also to the depressed state of physiological activity.
EFFECT OF AGE.
In a Mimosa plant, different leaves will be found of different age. Of these the youngest will be at the top. Lower down, we obtain a fully grown young leaf, and near the base, leaves which are very old. The investigation deals with the effect of age on the conducting power of the petiole.
Comparison of conducting power in different leaves: Experiment 34.—Selecting three leaves from the same plant we apply an identical electric stimulus at points 2 cm. from the three responding pulvini. The electric connections are so made that the same tetanising shock is applied on the three petioles, very young, fully grown, and very old. The secondary coil is gradually pushed in till the leaves exhibit responsive fall. The fully grown leaf was the first to respond, the velocity of transmission being 23 mm. per second. The secondary coil had to be pushed nearer the primary through 6 cm. before excitation could be effectively transmitted through the young petiole; for the oldest leaf still stronger stimulus was necessary, since in this case the secondary had to be pushed through an additional distance of 4 cm. for effective transmission of excitation. I also determined the relative values of the minimal intensity of stimulus, effective in causing transmission of excitation in the three cases. Adopting as before the intensity of electric stimulus which causes bare perception in a human being as the unit, I find that the effective stimulus for a fully grown young petiole is 0.3 unit, while the very young required 2.5 units, and the very old 5 units. Hence it may be said that the conducting power of a very young is an eighth, and of the very old one-sixteenth of the conductivity of the fully grown young specimen.
It will thus be seen that the conducting power of a very young petiole is feebler than in a fully grown specimen. The conducting tissue, it is true, is present, but the power of conduction has not become fully developed. This power is, as we shall see later, conferred by the stimulus of the environment. In a very old specimen the diminution of conducting power is due to the general physiological decline.
EFFECT OF DESICCATION ON CONDUCTING TISSUES.
I have already shown that transmission in the plant is a process fundamentally similar to that taking place in the animal nerve; it has also been shown that the effects of various physical and chemical agents are the same in the conducting tissues of plant and of animal.
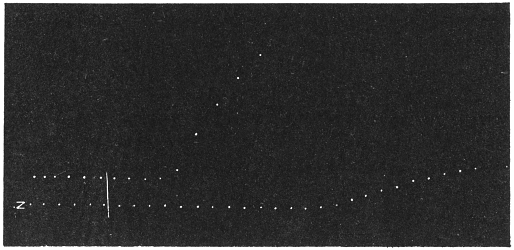
Fig. 41—Action of glycerine in enhancing the speed and intensity of transmitted excitation. Stimulus applied at the vertical line. Successive dots in record are at intervals of 0.1 sec.
Effect of application of glycerine: Experiment 35.—It is known that desiccation, generally speaking, enhances the excitability of the animal nerve. As glycerine, by absorption of water, causes partial desiccation, I tried its effect on conduction of excitation in the petiole of Mimosa. Enhancement of conducting power may be exhibited in two ways: first, by an increase of velocity of transmission; and, secondly, by an enhancement of the intensity of the transmitted excitation, which would give rise to a greater amplitude of response of the motile indicator. In Fig. 41 are given two records, N, before, and the other after the application of glycerine on a length of petiole through which excitation was being transmitted. The time-records demonstrate conclusively the enhanced rate of transmission after the application of glycerine. The increased intensity of transmitted excitation is also seen in the enhanced amplitude of response seen in the more erect curve in the upper record.
INFLUENCE OF TONIC CONDITION ON CONDUCTIVITY.
Different specimens of Mimosa are found to exhibit differences in physiological vigour. Some are in an optimum condition, others in an unfavourable or sub-tonic condition. I shall now describe certain characteristic differences of conductivity exhibited by tissues in different conditions.
Effect of intensity of stimulus on velocity of transmission.—In a specimen at optimum condition, the velocity remains constant under varying intensities of stimulus. Thus the velocity of transmission in a specimen was determined under a stimulus intensity of 0.5 unit; the next determination was made with a stimulus of four times the previous intensity, i.e., 2 units. In both these cases the velocity remained constant. But when the specimen is in a sub-tonic condition, the velocity is found to increase with the intensity of the stimulus. Thus the velocity of conduction of a specimen of Mimosa in a sub-tonic condition was found to be 5.9 mm. per second under a stimulus of 0.5 unit; with the intensity raised to 2.5 units, the velocity was enhanced to 8.3 mm. per second.
After-effect of stimulus.—In experimenting with a particular specimen of Mimosa I found that on account of its sub-tonic condition, the conducting power of the petiole was practically absent. Previous stimulation was, however, found to confer the power of conduction as an after-effect. It is thus seen that stimulus canalises a path for conduction.
The effect of excessive stimulus in a specimen in an optimum condition is to induce a temporary depression of conductivity; the effect of strong stimulus on a sub-tonic specimen is precisely the opposite, namely, an enhancement of conductivity. I give below accounts of two typical experiments carried out with petiole-pulvinus preparation of Mimosa. Excessive stimulation in these cases was caused by injury.
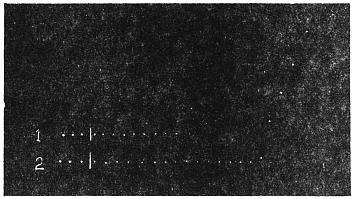
Fig. 42.—Effect of injury, depressing rate of conduction in normal specimen; (1) record before, and (2) after injury. (Dot-intervals, 0.1 sec.).
Action of Injury on Normal Specimens: Experiment 36.—A cut stem with entire leaf was taken, and stimulus applied at a distance of 15 mm. from the pulvinus. From the normal record (1) in Fig. 42 the velocity of transmission was found to be 18.7 mm. per sec. The end of the petiole beyond the point of application of the testing stimulus was now cut off, and record of velocity of transmission taken once more. It will be seen from record (2) that the excessive stimulus caused by injury had induced a depression in the conducting power, the velocity being reduced to 10.7 mm. per sec. Excessive stimulation of normal specimens is thus seen to depress temporarily the conducting power.
Action of Injury on Sub-tonic Specimens: Experiment 37.—I will now describe a very interesting experiment which shows how an identical agent may, on account of difference in the tonic condition of the tissue, give rise to diametrically opposite effects. In demonstrating this, I took a specimen in a sub-tonic condition, in which the conducting power of the tissue was so far below par, that the test-stimulus applied at a distance of 15 mm. failed to be transmitted (Fig. 43). The end of the petiole at a distance of 1 cm. beyond the point of application of test-stimulus was now cut off. The after-effect of this injury was found to enhance the conducting power so that the stimulus previously arrested was now effectively transmitted, the velocity being 25 mm. per sec. This enhanced conducting power began slowly to decline, and after half an hour the velocity had declined to 4.1 mm. per sec. The end of the petiole was cut once more, and the effect of injury was again found to enhance the conducting power, the velocity of transmission being restored to 25 mm. per sec.
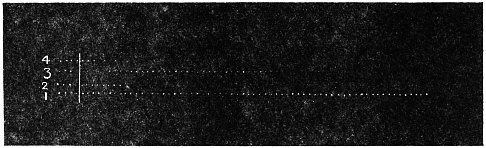
Fig. 43.—Effect of injury in enhancing the conducting power of a sub-normal specimen; (1) Ineffective transmission becoming effective at (2) after section; (3) decline after half an hour, and (4) increased conductivity after a fresh cut.
SUMMARY.
There are two different types of propagation of excitation: by convection, and by conduction. In the former the excited cell undergoes deformation and causes mechanical stimulation of the next; example of this type is seen in the stamen of Berberis. The conduction of excitation consists, on the other hand, of propagation of excitatory protoplasmic change. The transmission in the petiole of Mimosa is a phenomenon of conduction.
This conduction takes place along vascular elements. The conductivity is very much greater in the longitudinal than in the transverse direction.
Rise of temperature enhances, and fall of temperature lowers, the rate of conduction. Excitation is transmitted in both directions; the centrifugal velocity is greater than the centripetal.
Dessication of conducting tissue by glycerine enhances the conducting power. Local application of cold depresses or arrests the conduction. Application of poison permanently abolishes the power of conduction.
Conductivity is modified by the effect of season, being higher in summer than in winter.
The power of conduction is also modified by age. In young specimens the conducting power is low, the conductivity is at its maximum in fully grown organs; but a decline of conductivity sets in with age.
The tonic condition of a tissue has an influence on conductivity. In an optimum condition, the velocity is the same for feeble or strong stimulus. Excessive stimulation induces a temporary depression of the conducting power.
The effects are different in a sub-tonic tissue: velocity of transmission increases with intensity of stimulus; after-effect of stimulus is to initiate or enhance the conducting power. The conducting path is canalised by stimulus.
VII.—ON ELECTRIC CONTROL OF EXCITATORY IMPULSE
By
Sir J. C. Bose.
I have in my previous works[L] described investigations on the conduction of excitation in Mimosa pudica. It was there shown that the various characteristics of the propagation of excitation in the conducting tissue of the plant are in every way similar to those in the animal nerve. Hence it appeared probable that any newly found phenomenon in the one case was likely to lead to discovery of a similar phenomenon in the other.
As the transmission of excitation is a phenomenon of propagation of molecular disturbance in the conducting vehicle, it appeared that the excitatory impulse could be controlled by inducing in the conducting tissue two opposite ‘molecular dispositions’, using that term in the widest sense. The possibility of accomplishing this by the directive action of an electric current had attracted my attention for many years.
METHOD OF CONDUCTIVITY BALANCE.
I have previously carried out an electric method of investigation, dealing with the influence of electric current on conductivity. The method of Conductivity Balance which I devised for this purpose[M] was found very suitable. Isolated conducting tissues of certain plants were found to exhibit transmitted effect of excitatory electric change of galvanometric negativity, which at the favourable season of the year was of sufficient intensity to be recorded by a sensitive galvanometer. A long strand of the conducting tissue was taken and two electric connections were made with a galvanometer, a few centimetres from the free ends. Thermal stimulus was applied at the middle, when two excitatory waves with their concomitant electric changes were transmitted outwards. By suitably moving the point of application of stimulus nearer or further away from one of the two electric contacts, an exact balance was obtained. This was the case when the resultant galvanometer deflection was reduced to zero. If now an electrical current be sent along the length of the conducting tissue, the two excitatory waves sent outwards from the central stimulated point will encounter the electric current in different ways; one of the excitatory waves will travel with, and the other against the direction of the current. If the power of transmitting excitation is modified by the direction of an electric current then the magnitudes of transmitted excitations will be different in the two cases, with the result of the upsetting of the Conductivity Balance. From the results of experiments carried out by this method on the effect of feeble current on conductivity, the conclusion was arrived at that excitation is better conducted against the direction of the current than with it. In other words, the influence of an electric current is to confer a preferential or selective direction of conductivity for excitation, the tissue becoming a better conductor in an electric up-hill direction compared with a down-hill.
The results were so unexpected that I have for long been desirous of testing the validity of this conclusion by independent method of inquiry. I shall presently give full account of the perfected method, and the various difficulties which had to be overcome to render it practical. Before doing this I shall describe a simple method which I have devised for demonstrating the principal results.
CONTROL OF TRANSMITTED EXCITATION IN AVERRHOA BILIMBI.
The petiole of Averrhoa bilimbi has a large number of paired leaflets, which, on excitation, undergo downward closure. Feeble stimulus is applied at a point in the petiole, and the transmission of excitation is visibly manifested by the serial fall of the leaflets. The distance to which the excitation reaches is a measure of normal power of conduction. Any variation of conductivity, by the passage of an electric current in one direction or the other is detected by the enhancement or diminution of the distance through which excitation is transmitted. I shall describe the special precautions to be taken in carrying out this investigation.
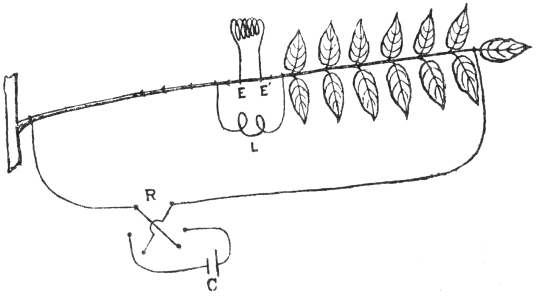
Fig. 44.—Diagram of experimental arrangement for control of transmitted excitation in Averrhoa bilimbi. For explanation see text.
Electric stimulus of induction shock of definite intensity and duration is supplied at the middle of the petiole at EE′ (Fig. 44). The leaflets to the left of E, are not necessary for the purpose of this experiment and therefore removed. The intensity of the induction shock may be varied in the usual manner by removing the secondary coil nearer or farther from the primary. The duration of the shock is always maintained constant. On application of electric stimulus excitation is transmitted along the petiole, the distance of transmission depending on the intensity of stimulus. With feeble stimulus two pairs of leaflets may undergo an excitatory fall; with stronger stimulus the transmission is extended to the end of the petiole, and all the leaflets exhibit movements of closure. We shall now study the modifying influence of a constant current on conduction of excitation. C is an electric cell, R the reversing key by which the electric current could be sent from right to left or in the opposite direction. When the current is sent from right to the left, the excitatory impulse initiated at EE′ travels against the direction of the current in an ‘up-hill’ direction. When the current is reversed it flows in the petiole from left to right and the transmitted impulse travels with the current or in a ‘down-hill’ direction.
Two complications are introduced on the completion of the electric circuit of the constant current: the first, is the distributing effect of leakage of the induction current used for excitation, and second, the polar variation of excitation induced by the constant current.
Leakage of induction current.—Before completing the constant current circuit, the alternating induction current goes only through the path EE′. On completion of the constant current circuit, the alternating induction current not only passes through the shorter path EE′ but also by the circuitous path of the constant current circuit. The escaping induction current would thus excite all the leaflets directly and not by its transmitted action. This difficulty is fully overcome by the interposition of a choking coil which will be described below. A simpler, though less perfect, device may be employed to reduce and practically eliminate the leakage. This consists of a loop, L, of silver wire placed outside EE′. The leakage of induction current is thus diverted along this path of negligible resistance in preference to the longer circuit through the entire petiole, which has a resistance of several million ohms.
Polar action of current on excitability.—It is well known that an electric current induces a local depression of excitability at the point of entrance to the tissue, or at the anode, and an enhancement of excitability at the point of exit, or at the cathode. But the excitability is unaffected at a point equally distant from anode and cathode. This is known as the indifferent point. The exciting electrodes EE′ are placed at the indifferent point. But when the current enters on the right side, the terminal leaflets to the right have their excitability depressed by the proximity of anode, but the leaflets near the electrodes EE′, being at a distance from the anode are not affected by it. Moreover it will be shown that the enhanced conductivity conferred by the directive action of the current overpowers any depression of excitability in the terminal leaflets due to the proximity of the anode. I shall, for convenience, designate the transmission as ‘up-hill’, when excitation is propagated against the direction of the constant electric current, and ‘down-hill’ when transmitted with the direction of the current.
Transmission of excitation ‘Up-hill’: Experiment 38.—I shall give here an account of an experiment which may be taken as typical. I took a vigorous specimen of Averrhoa bilimbi, and applied a stimulus whose intensity was so adjusted that the propagated impulse brought about a fall of only two pairs of leaflets. This gave a measure of normal conduction without the passage of the current. The constant electric current was now sent from right to left. A necessary precaution is to increase the current gradually by means of a suitable potentiometer slide, to its full value. The reason for this will be given later. The intensity of the constant current employed was 1.4 micro-ampères. Now on exciting the petiole by the previous stimulus, the conducting power was found to be greatly enhanced. The excitatory impulse now reached the end of the petiole, and caused six pairs of leaflets to fall.
Transmission of excitation ‘Down-hill’: Experiment 39.—In continuation of the previous experiment, the constant electric current was reversed, its directions being now from left to right. Transmission of excitation was now in a down-hill direction. On applying the induction shock stimulus of the same intensity as before, the conducting power of the petiole was found to be abolished, none of the leaflets exhibiting any sign of excitation. This modification of the conducting power persists during the passage of the constant current. On cessation of the current the original conducting power is found to be restored. It will thus be seen that the power of conduction is capable of modification, and that the passage of an electric current of moderate intensity induces enhanced power of conduction in an ‘up-hill’ and diminished conductivity in a ‘down-hill’ direction.
ELECTRIC CONTROL OF NERVOUS IMPULSE IN ANIMALS.
In my ‘Researches on Irritability of Plants’ I have shown how intimately connected are the various physiological reactions in the plant and in the animal, and I ventured to predict that the recognition of this unity of response in plant and animal will lead to further discoveries in physiology in general. This surmise has been fully justified, as will be seen in the following experiments carried out on the nerve-and-muscle preparation of a frog. It is best to carry out the experiments with vigorous specimens; this ensures success, even in long continued experiments, which can then be repeated with unfailing certainty for hours. It is also an advantage to use a large frog for its relatively great length of the nerve.
Directive action of current on conduction of excitation in a nerve-and-muscle preparation: Experiment 40.—A preparation was made with a length of the spine and two nerves leading to the muscles. The specimen is supported in a suitable manner, and electric connections made with the toes, one for the entrance and the other for exit of the constant current. The current thus entered, say, by the left toe ascended the muscle and went up the nerve on the left side, and descended through the other nerve on the right side along the muscle and thence to the right toe. Before the passage of the constant electric current the spinal nerve was stimulated by an induction shock of definite intensity. The nervous impulse was conducted by the two nerves, one to the left and the other to the right, and caused a feeble twitch of the respective muscles. A feeble current of 1.5 micro-ampère was sent along the nerve-and-muscle circuit, ascending by the left and descending by the right side. It will be seen that excitation initiated at the spine is propagated ‘against’ the electric current on the left side, and ‘with’ the current on the right side. On repetition of previous electric stimulus the effect of directive action of current was at once manifested by the left limb being thrown into a state of strong tetanic contraction, whereas the right limb remained quiescent. By changing the direction of the constant current the induced enhancement of conductivity of the nerve was quickly transferred from the left to the right side, the depression or arrest of conduction being simultaneously transferred to the left side. Turning the reversing key one way or the other brought about supra or non-conducting state of the nerve, and this condition was maintained throughout the duration of the current.
I shall next describe a more perfect method for obtaining quantitative results both with plant and animal. In order to demonstrate the universality of the phenomenon, I next used Mimosa pudica instead of Averrhoa, for experiments on plants.
For determination of normal velocity of transmission of excitation and the induced variation of that velocity, I employed the automatic method of recording the velocity of transmission of excitation in Mimosa, where the excitatory fall of the motile leaf gave a signal for the arrival of the excitation initiated at a distant point. In this method the responding leaf is attached to a light lever, the writer being placed at right angles to it. The record is taken on a smoked glass plate, which during its descent makes an instantaneous electric contact, in consequence of which a stimulating shock is applied at a given point of the petiole. A mark in the recording plate indicates the moment of application of stimulus. After a definite interval the excitation is conducted to the responding pulvinus, when the excitatory fall of the leaf pulls the writer suddenly to the left. From the curve traced in this manner the time-interval between the application of stimulus and the initiation of response can be found, and the normal rate of transmission of excitation through a given length of the conducting tissue deduced. The experiment is then repeated with an electric current flowing along the petiole with or against the direction of transmission of excitation. The records thus obtained enable us to determine the influence of the direction of the current on the rate of transmission. I shall presently describe the various difficulties which have to be overcome before the method just indicated can be rendered practical.
The scope of investigation will be best described according to the following plan[N]:—
PART I.—INFLUENCE OF DIRECTION OF ELECTRIC CURRENT ON CONDUCTION OF EXCITATION IN PLANTS.
General method of experiment.
Effect of feeble current on velocity of transmission of excitation ‘up-hill’ or ‘down-hill.’
Determination of variation of conductivity by the method of minimal stimulus and response.
The after-effect of current.
PART II.—INFLUENCE OF DIRECTION OF ELECTRIC CURRENT ON CONDUCTION OF EXCITATION IN ANIMAL NERVE.
The method of experiment.
Variation of velocity of transmission under the action of current.
Variation in the intensity of transmitted excitation.
PART I.—INFLUENCE OF DIRECTION OF CURRENT ON TRANSMISSION OF EXCITATION IN PLANT.
THE METHOD OF EXPERIMENT.
I may here say a few words of the manner in which the period of transmission can be found from the record given by my Resonant Recorder, fully described in my previous paper. The writer attached to the recording lever of this instrument is maintained by electromagnetic means in a state of to-and-fro vibration. The record thus consists of a series of dots made by the tapping writer, which is tuned to vibrate at a definite rate, say, 10 times per second. In a particular case whose record is given in Curve 1 (Fig. 46), indirect stimulus of electric shock was applied at a distance of 15 mm. from the responding pulvinus. There are 15 intervening dots between the moment of application of stimulus and the beginning of response; the time-interval is therefore 1.5 seconds. The latent period of the motile pulvinus is obtained from a record of direct stimulation; the average value of this in summer is 0.1 second. Hence the true period of transmission is 1.4 seconds for a distance of 15 mm. The velocity determined in this particular case is therefore 10.7 mm. per second.
Precaution has to be taken against another source of disturbance, namely, the excitation caused by the sudden commencement or the cessation of the constant current. I have shown elsewhere[O] that the sudden initiation or cessation of the current induces an excitatory reaction in the plant-tissue similar to that in the animal tissue. This difficulty is removed by the introduction of a sliding potentiometer, which allows the applied electromotive force to be gradually increased from zero to the maximum or decreased from the maximum to zero.
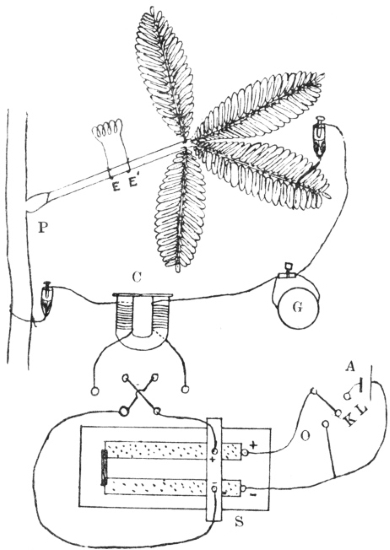
Fig. 45.—Complete apparatus for investigation of the variation of conducting power in Mimosa. A, storage cell; S, potentiometer slide, which, by alternate movement to right or left, continuously increases or decreases the applied E.M.F.; K, switch key for putting current “on” and “off” without variation of resistance; E, E′, electrodes of induction coil for stimulation; C, choking coil; G, micro-ammeter.
The experimental arrangement is diagrammatically shown in Fig. 45. After attaching the petiole to the recording lever, indirect stimulus is applied, generally speaking, at a distance of 15 mm. from the responding pulvinus. Stimulus of electric shock is applied in the usual manner, by means of a sliding induction coil. The intensity of the induction shock is adjusted by gradually changing the distance between the secondary and the primary, till a minimally effective stimulus is found. In the study of the effect of direction of constant current on conductivity, non-polarisable electrodes make suitable electric connections, one with the stem and the other with the tip of a sub-petiole at a distance from each other of about 95 mm. The point of stimulation and the responding pulvinus are thus situated at a considerable distance from the anode or the cathode, in the indifferent region in which there is no polar variation of excitability. By means of a Pohl’s commutator or reverser, the constant current can be maintained either “with” or “against” the direction of transmission of excitation. The transmission in the former case is “down-hill,” and in the latter case “up-hill.” Electrical connections are so arranged that when the commutator is tilted to the right, the transmission is down-hill, when tilted to the left, up-hill.
The electrical resistance offered by the 95 mm. length of stem and petiole will be from two to three million ohms. The intensity of the constant current flowing through the plant can be read by unplugging the key which short-circuits the micro-ammeter G. The choking coil C prevents the alternating induction current from flowing into the polarising circuit and causing direct stimulation of the pulvinus.
Before describing the experimental results, it is as well to enter briefly into the question of the external indication by which the conducting power may be gauged. Change of conductivity may be expected to give rise to a variation in the rate of propagation or to a variation in the magnitude of the excitatory impulse that is transmitted. Thus we have several methods at our disposal for determining the induced variation of conductivity. In the first place the variation of conductivity may be measured by the induced change in the velocity of transmission of excitation. In the second place, the transmitted effect of a sub-maximal stimulus will give rise to enhanced or diminished amplitude of mechanical response, depending on the increase or decrease of conductivity brought about by the directive action of the current. And, finally, the enhancement or depression of conductivity may be demonstrated by the ineffectively transmitted stimulus becoming effective, or the effectively transmitted stimulus becoming ineffective.
Exclusion of the factor of Excitability.—The object of the enquiry being the pure effect of variation of conductivity, we have to assure ourselves that under the particular conditions of the experiment the complicating factor of polar variation of excitability is eliminated. It is to be remembered that excitatory transmission in Mimosa takes place by means of a certain conducting strand of tissue which runs through the stem and the petiole. In the experiment to be described, the constant current enters by the tip of the petiole and leaves by the stem, or vice versâ, the length of the intrapolar region being 95 mm. The point of application of stimulus on the petiole is 40 mm. from the electrode at the tip of the leaf. The responding pulvinus is also at the same distance from the electrode on the stem. The point of stimulation and region of response are thus at the relatively great distance of 40 mm. from either the anode or the cathode, and may therefore be regarded as situated in the indifferent region. This is found to be verified in actual experiments.
EFFECTS OF DIRECTION OF CURRENT ON VELOCITY OF TRANSMISSION.
A very convincing method of demonstrating the influence of electric current on conductivity consists in the determination of changes induced in the velocity of transmission by the directive action of the current. For this purpose we have to find out the true time required by the excitation to travel through a given length of the conducting tissue (1) in the absence of the current, (2) ‘against’ and (3) ‘with’ the direction of the current. The true time is obtained by subtracting the latent period of the pulvinus from the observed interval between the stimulus and response. Now the latent period may not remain constant, but undergo change under the action of the polarising current. It has been shown that the excitability of the pulvinus does not undergo any change when it is situated in the middle or indifferent region. The following results show that under parallel conditions the latent period also remains unaffected:—
TABLE V.—SHOWING THE EFFECT OF ELECTRIC CURRENT ON THE LATENT PERIOD.
SpecimensI.II.
sec.sec.
Latent period under normal condition0.100.09
" " " current from right to left0.110.10
" " " current from left to right0.090.09
The results of experiments with two different specimens given above show that a current applied under the given conditions has practically no effect on the latent period, the slight variation being of the order of one-hundredth part of a second. This is quite negligible when the total period observed for transmission is, as in the following cases, equal to nearly 2 seconds.
Induced changes in the Velocity of Transmission.—Having found that the average value of the latent period in summer is 0.1 second, we next proceed to determine the influence of the direction of current on velocity.
Experiment 41.—As a rule, stimulus of induction shock was applied in this and in the following experiments on the petiole at a distance of 15 mm. from the responding pulvinus. The recording writer was tuned to 10 vibrations per second; the space between two succeeding dots, therefore, represents a time-interval of 0.1 second. The middle record, N in Fig. 46, is the normal. There are 17 spaces between the application of stimulus and the beginning of response. The total time is therefore 1.7 seconds, and by subtracting from it the latent period of 0.1 second we obtain the true time, 1.6 seconds. The normal velocity is found by dividing the distance 15 mm. by the true interval 1.6 seconds. Thus V = 1 5/1.6 = 9.4 mm. per second. We shall next consider the effect of current in modifying the normal velocity. The uppermost record (1) in Fig. 46 was taken under the action of an ‘up-hill,’ or ‘against’ current of the intensity of 1.4 microampères. It will be seen that the time interval is reduced from 1.7 seconds to 1.4 seconds; making allowance for the latent period, the velocity of transmission under ‘up-hill’ current V1 = 1 5/1.3 = 11.5 mm. per second. In the lowest record (3) we note the effect of ‘down-hill’ current, the time-interval between stimulus and response being prolonged to 1.95 seconds and the velocity reduced to 8.1 mm. per second. The conclusion arrived at from this mechanical mode of investigation is thus identical with that derived from the electric method of conductivity balance referred to previously.
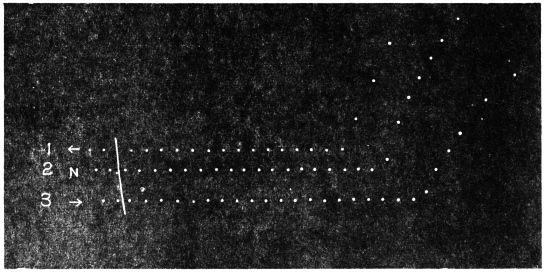
Fig. 46.—Record showing enhancement of velocity of transmission “up-hill” or against the current (uppermost curve) and retardation of velocity “down-hill” or with the current (lowest curve). N, normal record in the absence of current; ← indicates “up-hill” and → “down-hill” transmission.
That is to say, the passage of a feeble current modifies conductivity for excitation in a selective manner. Conductivity is enhanced against, and diminished with, the direction of the current.
The minimum current which induces a perceptible change of conductivity varies somewhat in different specimens. The average value of this minimal current in autumn is 1.4 microampères. The effect of even a feebler current may be detected by employing a test stimulus which is barely effective.
TABLE VI.—SHOWING EFFECTS OF UP-HILL AND DOWN-HILL CURRENTS OF FEEBLE INTENSITY ON PERIOD OF TRANSMISSION THROUGH 15 MM.
Number.Intensity of current in microampères.Period for up-hill transmission.Period for down-hill transmission.
11.414 tenths of a second16 tenths of a second
21.413 " "15 " "
31.619 " "Arrest.
41.712 " "14 tenths of a second
Having demonstrated the effect of direction of current on the velocity of transmission, I shall next describe other methods by which induced variations of conductivity may be exhibited.
DETERMINATION OF VARIATION OF CONDUCTIVITY BY METHOD OF MINIMAL STIMULUS AND RESPONSE.
In this method we employ a minimal stimulus, the transmitted effect of which under normal conditions gives rise to a feeble response. If the passage of a current in a given direction enhances conductivity, then the intensity of transmitted excitation will also be enhanced; the minimal response will tend to become maximal. Or excitation which had hitherto been ineffectively transmitted will now become effectively transmitted. Conversely, depression of conductivity will result in a diminution or abolition of response. We may use a single break-shock of sufficient intensity as the test stimulus. It is, however, better to employ the additive effect of a definite number of feeble make-and-break shocks.
We may again employ additive effect of a definite number of induction shocks, the alternating elements of which are exactly equal and opposite. This is secured by causing rapid reversals of the primary current by means of a rotating commutator. The successive induction shocks of the secondary coil can thus be rendered exactly equal and opposite.
Experiment 42.—Working in this way, it is found that the transmitted excitation against the direction of current becomes effective or enhanced under ‘up-hill’ current. A current, flowing with the direction of transmission, on the other hand, diminishes the intensity of transmitted excitation or blocks it altogether.
Henceforth it would be convenient to distinguish currents in the two directions: the current in the direction of transmission will be distinguished as Homodromous, and against the direction of transmission as Heterodromous.
AFTER-EFFECTS OF HOMODROMOUS AND HETERODROMOUS CURRENTS.
The passage of a current through a conducting tissue in a given direction causes, as we have seen, an enhanced conductivity in an opposite direction. We may suppose this to be brought about by a particular molecular arrangement induced by the current, which assisted the propagation of the excitatory disturbance in a selected direction. On the cessation of this inducing force, there may be a rebound and a temporary reversal of previous molecular arrangement, with concomitant reversal of the conductivity variation. The immediate after-effect of a current flowing in a particular direction on conductivity is likely to be a transient change, the sign of which would be opposite to that of the direct effect. The after-effect of a heterodromous current may thus be a temporary depression, that of a homodromous current, a temporary enhancement of conductivity.
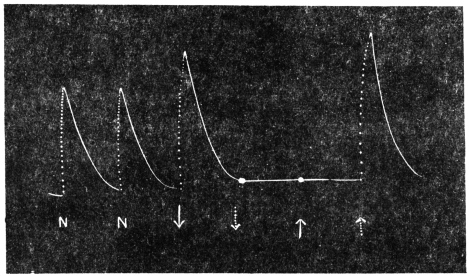
Fig. 47.—Direct and after-effect of heterodromous and homodromous currents. First two records, N, N, normal. ↓, enhanced transmission under heterodromous current; ⇣ arrest of conduction is an after-effect of heterodromous current. Next record ↑ shows arrest under homodromous current. Last record ⇡ shows enhancement of conduction greater than normal, as an after-effect of homodromous current. (Dotted arrow indicates the after-effect on cessation of a given current. ↑ homodromous and ↓ heterodromous current.)
Experiment 43.—This inference will be found fully justified in the following experiment:—The first two responses are normal, after which the heterodromous current gave rise to an enhanced response. The depressing after-effect of a heterodromous current rendered the next response ineffective. The following record taken during the passage of the homodromous current exhibited an abolition of response due to induced depression of conductivity. Finally, the after-effect of the homodromous current is seen to be a response larger than the normal (Fig. 47). These experiments show that the after-effect of cessation of a current in a given direction is a transient conductivity variation, of which the sign is opposite to that induced by the continuation of the current.
PART II—INFLUENCE OF DIRECTION OF ELECTRIC CURRENT ON CONDUCTION OF EXCITATION IN ANIMAL NERVE.
I shall now take up the question whether an electric current induced any selective variation of conductivity in the animal nerve, similar to that induced in the conducting tissue of the plant.
THE METHOD OF EXPERIMENT.
In the experiments which I am about to describe, arrangements were specially made so that (1) the excitation had not to traverse the polar region, and (2) the point of stimulation was at a relatively great distance from either pole. The fulfilment of the latter condition ensured the point of stimulation being placed at the neutral region.
In the choice of experimental specimens I was fortunate enough to secure frogs of unusually large size, locally known as “golden frogs” (Rana tigrina). A preparation was made of the spine, the attached nerve, the muscle and the tendon. The electrodes for constant current were applied at the extreme ends, on the spine and on the tendon (Fig. 48). The following are the measurements, in a typical case, of the different parts of the preparation. Length of spine between the electrode and the nerve = 40 mm. length of nerve = 90 mm. length of muscle = 50 mm. length of tendon = 30 mm. Stimulus is applied in all cases on the nerve, midway between the two electrodes this point being at a minimum distance of 100 mm. from either electrode. The point of stimulation is, therefore, situated at an indifferent region.
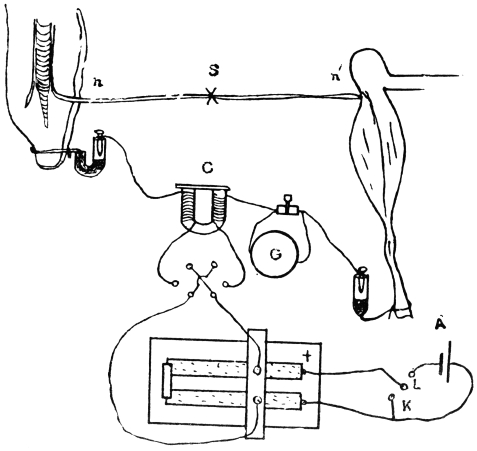
Fig. 48.—Experimental arrangement for study of variation of conductivity of nerve by the directive action of an electric current. n n′, nerve; S, point of application of stimulus in the middle or indifferent region.
Great precautions have to be taken to guard against the leakage of current. The general arrangement for the experiment on animal nerve is similar to that employed for the corresponding investigations on the plant. The choking coil is used to prevent the stimulating induction current from getting round the circuit of constant current. The specimen is held on an ebonite support, and every part of the apparatus insulated with the utmost care.
VARIATION OF VELOCITY OF TRANSMISSION.
In the case of the conducting tissue of the plant a very striking proof of the influence of the direction of current on conductivity was afforded by the induced variation of velocity of transmission. Equally striking is the result which I have obtained with the nerve of the frog.
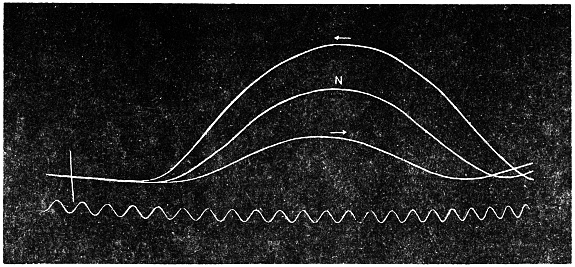
Fig. 49.—Effect of heterodromous and homodromous current in inducing variation in velocity of transmission through nerve. N, normal record, upper record shows enhancement, and lower record retardation in velocity of transmission under heterodromous and homodromous currents, respectively.
Experiment 44.—The experiments described below were carried out during the cold weather. The following records (Fig. 49), obtained by means of the pendulum myograph, exhibit the effect of the direction of current on the period of transmission through a given length of nerve. The latent period of muscle being constant, the variations in the records exhibit changed rates of conduction. The middle record is the normal, in the absence of any current. The upper record, denoted by the left-hand arrow, shows the action of a heterodromous current in shortening the period of transmission and thus enhancing the velocity above the normal rate. The lower record, denoted by the right-hand arrow, exhibits the effect of a homodromous current in retarding the velocity below the normal rate. I find that a very feeble heterodromous current is enough to induce a considerable increase of velocity, which soon reaches a limit. For inducing retardation of velocity, a relatively strong homodromous current is necessary. I give below a table showing the results of several experiments.
TABLE V—EFFECT OF HETERODROMOUS AND HOMODROMOUS CURRENT OF FEEBLE INTENSITY ON VELOCITY OF TRANSMISSION.
Specimen.Intensity of heterodromous current.Acceleration above normal.Intensity of homodromous current.Retardation below normal.
microampèreper cent.microampèresper cent.
10.35161.020
20.70131.519
30.80182.014
40.80112.013
51.00182.512
61.50153.040
VARIATION OF INTENSITY OF TRANSMITTED EXCITATION UNDER HETERODROMOUS AND HOMODROMOUS CURRENTS.
In the next method of investigation, the induced variation of intensity of transmitted excitation is inferred from the varying amplitude of response of the terminal muscle. Testing stimulus of sub-maximal intensity is applied at the middle of the nerve, where the constant current induces no variation of excitability. Stimulation is effected either by single break-shock or by the summated effects of a definite number of equi-alternating shocks, or by chemical stimulation
Experiment 45.—Under the action of feeble heterodromous current the transmitted excitation was always enhanced, whatever be the form of stimulation. This is seen illustrated in Fig. 50. Homodromous current on the other hand inhibited or blocked excitation (Fig. 51).
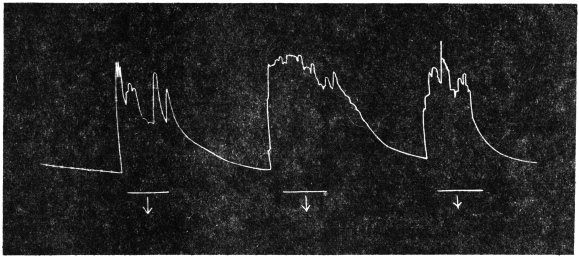
Fig. 50.—Ineffectively transmitted salt-tetanus becoming effective under heterodromous current, denoted by down-pointing arrow.
Complication due to variation of Excitability of Muscle.—In experiments with the plant, there was the unusual advantage in having both the point of stimulation and the responding motile organ in the middle or indifferent region. Unfortunately this ideally perfect condition cannot be secured in experiments with the nerve-and-muscle preparation of the frog. It is true that the point of stimulation in this case is chosen to lie on the nerve at the middle or indifferent region. But the responding muscle is at one end, not very distant from the electrode applied on the tendon. It is, therefore, necessary to find out by separate experiments any variation of excitability that might be induced in the muscle by the proximity of either the anode or the cathode, and make allowance for such variation in interpreting the results obtained from investigations on variation of conductivity.
In the experimental arrangement employed, the heterodromous current is obtained by making the electrode on the spine cathode and that on the tendon anode. The depressing influence of the anode in this case may be expected to lower, to a certain extent, the normal excitability of the responding muscle. Conversely, with homodromous current, the tendon is made the cathode and under its influence the muscle might have its excitability raised above the normal. These anticipations are fully supported by results of experiments. Sub-maximal stimulus of equi-alternating induction shock was directly applied to the muscle and records taken of (1) response under normal condition without any current, (2) response under heterodromous current, the tendon being the anode, and (3) response under homodromous current, the tendon being now made the cathode. It was thus found that under heterodromous current the excitability of the muscle was depressed, and under homodromous current the excitability was enhanced.
The effect of current on response to direct stimulation is thus opposite to that on response to transmitted excitation, as will be seen in the following Table.
TABLE VIII.—INFLUENCE OF DIRECTION OF CURRENT ON DIRECT AND TRANSMITTED EFFECTS OF STIMULATION.
Direction of current.Transmitted excitation.Direct stimulation.
Heterodromous currentEnhanced responseDepressed response
Homodromous currentDepressed responseEnhanced response
The passage of a current, therefore, induces opposing effects on the conductivity of the nerve and the excitability of the muscle, the resulting response being due to their differential actions. Under heterodromous current a more intense excitation is transmitted along the nerve, on account of induced enhancement of conductivity. But this intense excitation finds the responding muscle in a state of depressed excitability. In spite of this the resulting response is enhanced (Fig. 50). The enhancement of conduction under heterodromous current is, in reality, much greater than is indicated in the record. Similarly, under homodromous current the depression of conduction in the nerve may be so great as to cause even an abolition of response, in spite of the enhanced excitability of the muscle (Fig. 51). The actual effects of current on conductivity are, thus, far in excess of what are indicated in the records.
AFTER-EFFECTS OF HETERODROMOUS AND HOMODROMOUS CURRENTS.
On the cessation of a current there is induced in the plant-tissue a transient conductivity change of opposite sign to that induced by the direct current (cf. Expt. 43). The same I find to be the case as regards the after-effect of current on conductivity change in animal nerve. Of this I only give a typical experiment of the direct and after-effect of homodromous current on salt-tetanus.
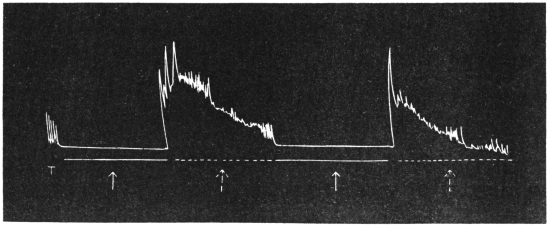
Fig. 51.—Direct and after-effect of homodromous current. Transmitted excitation (salt-tetanus T,) arrested under homodromous current denoted by up-pointing arrow; on cessation of current represented by dotted line there is a transient enhancement above the normal.
Experiment 46.—In this experiment sufficient length of time was allowed to elapse after the application of the salt on the nerve, so that the muscle, in response to the transmitted excitation, exhibited an incomplete tetanus T. The homodromous current was next applied, with the result of inducing a complete block of conduction, with the concomitant disappearance of tetanus. The homodromous current was gradually reduced to zero by the appropriate movement of the potentiometer slide. The after-effect of homodromous current is now seen in the transient enhancement of transmitted excitation, which lasted for nearly 40 seconds. After this the normal conductivity was restored. Repetition of the experiment gave similar results (Fig. 51).
The results that have been given are only typical of a very large number, which invariably supported the characteristic phenomena that have been described.
It will thus be seen that with feeble or moderate current, conductivity is enhanced against the direction of the current and depressed or blocked with the direction of the current. Under strong current the normal effect is liable to undergo a reversal.
It has thus been shown that a perfect parallelism exists in the conductivity variation induced in the plant and in the animal by the directive action of the current. No explanation could be regarded as satisfactory which is not applicable to both cases. Now with the plant we are able to arrange the experimental condition in such a way that the factor of variation of excitability is completely eliminated. The various effects described about the plant-tissue are, therefore, due entirely to variation of conductivity. The parallel phenomena observed in the case of transmission of excitation in the animal nerve must, therefore, be due to the induced change of conductivity.
The action of an electrical current in inducing variation of conductivity may be enunciated under the following laws, which are equally applicable to the conducting tissue of the plant and the nerve of the animal:—
LAWS OF VARIATION OF NERVOUS CONDUCTION UNDER THE ACTION OF ELECTRIC CURRENTS.
1. The passage of a current induces a variation of conductivity, the effect depending on the direction and intensity of current.
2. Under feeble intensity, heterodromous current enhances, and homodromous current depresses, the conduction of excitation.
3. The after-effect of a feeble current is a transient conductivity variation, the sign of which is opposite that induced during the continuation of current.
SUMMARY.
The variation of conductivity induced by the directive action of current has been investigated by two different methods:—
(1) The method in which the normal speed and its induced variation are automatically recorded;
(2) That in which the variation in the intensity of transmitted excitations is gauged by the varying amplitudes of resulting responses.
The great difficulty arising from leakage of the exciting induction current into the polarising circuit was successfully overcome by the interposition of a choking coil.
The following summarises the effects of direction and intensity of an electric current, on transmission of excitation through the conducting tissue of the plant.
The velocity of transmission is enhanced against the direction of a feeble current, and retarded in the direction of the current.
Feeble heterodromous current enhances conductivity, homodromous current, on the other hand, depresses it.
Ineffectively transmitted excitation becomes effectively transmitted under heterodromous current. Effectively transmitted excitation, on the other hand, becomes ineffectively transmitted under the action of homodromous current.
The after-effect of a current is a transient conductivity change, the sign of which is opposite to that induced during the passage of current. The after-effect of a heterodromous current is, thus, a transient depression, that of homodromous current, a transient enhancement of conductivity.
The characteristic variations of conductivity induced in animal nerve by the direction and intensity of current are in every way similar to those induced in the conducting tissue of the plant.
These various effects are demonstrated by the employment of not one, but various kinds of testing stimulus, such as the excitation caused (1) by a single break-induction shock or (2) by a series of equi-alternating tetanising shocks or (3) by chemical stimulation.
VIII.—EFFECT OF INDIRECT STIMULUS ON PULVINATED ORGANS
By
Sir J. C. Bose,
Assisted by
Guruprasanna Das, L.M.S.
The leaf of Mimosa pudica undergoes an almost instantaneous fall when the stimulus is applied directly on the pulvinus which is the responding organ. The latent period, i.e., the interval between the application of stimulus and the resulting response is about 0.1 second. Indirect stimulus, i.e., application of stimulus at a distance from the pulvinus, also causes a fall of the leaf; but a longer interval will elapse between the incidence of stimulus and the response; for it will take a definite time for the excitation to be conducted through the intervening tissue. I have already shown that this conduction of excitation in plant is analogous to the transmission of nervous impulse in animal.
The power of conduction varies widely in different plants. In the petiole of Mimosa pudica the velocity may be as high as 30 mm. per second. In the stem the velocity is considerably less, i.e., about 6 mm. per second in the longitudinal direction; but conduction across the stem is a very much slower process. In the petiole of Averrhoa the longitudinal velocity is of the order of 1 mm. per second.
DUAL CHARACTER OF THE TRANSMITTED IMPULSE.
The record of the transmitted effect of stimulus is found to exhibit a remarkable preliminary variation. This was detected by my delicate recorders, which gave magnifications from fifty to hundred times. I shall give a detailed account of a typical experiment carried out with Averrhoa carambola, which will bring out clearly the characteristic effects of Indirect Stimulus.
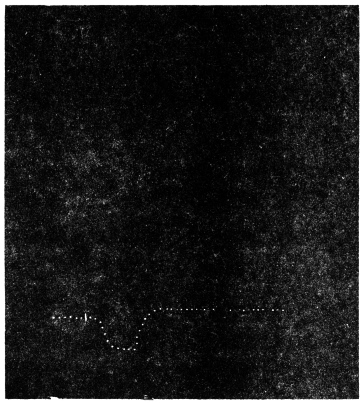
Fig. 52.—Effect of indirect Stimulus on leaflet of Averrhoa carambola. Stimulus was applied at the short vertical line. Successive dots at intervals of one second. Note the positive response preceding the negative.
Experiment 47.—Stimulus of electric shock applied at a point on the long petiole of Averrhoa causes successive fall of pairs of leaflets. In the experiment to be described one of the leaflets of the plant was attached to the recorder. Stimulus was applied at a distance of 50 mm. The successive dots in the record are at intervals of a second. It will be noticed that two distinct impulses—a positive and a negative—were generated by the action of Indirect Stimulus. The positive impulse reached the responding organ after 1.5 second and caused an erectile movement. The velocity of the positive impulse in the present case is 33 mm. per second. The normal excitatory negative impulse reached the motile organ 44 seconds after the application of stimulus, and caused a very rapid fall of the leaflet, the fall being far more pronounced than the positive movement of erection (Fig. 52). In this and in all subsequent records, the positive and negative responses offer a great contrast. The movement in response to positive reaction is slow, whereas that due to negative reaction is very abrupt, almost ‘explosive,’ the successive dots being now very wide apart. As regards the velocity of impulse the relation is reversed, the positive being the quicker of the two. In the present case, the velocity of the excitatory negative impulse is 1.1 mm. per second, as against 33 mm. of the positive impulse.
The negative impulse is due to the comparatively slow propagation of the excitatory protoplasmic change, which brings about a diminution of turgor in the pulvinus and fall of the responding leaflet. The erectile movement of the leaflet by the positive impulse must be due to an increase of turgor, brought on evidently, by the forcing in of water. This presupposes a forcing out of water somewhere else, probably at the point of application of stimulus. It may be supposed that an active contraction occurred in plant cells under direct stimulus, in consequence of which water was forced out giving rise to a hydraulic wave. On this supposition the positive impulse is to be regarded as hydro-mechanical. I have, however, not yet been able to devise a direct experimental test to settle the question.
EFFECT OF DISTANCE OF APPLICATION OF STIMULUS.
In the last experiment the stimulus was applied at the moderate distance of 50 mm. Let us now consider the respective effects, first, of an increase, and second, of a decrease of the intervening distance. In a tissue whose conducting power is not great, the excitatory impulse is weakened, even to extinction in transmission through a long distance. Thus the negative impulse may fail to reach the responding organ, when the stimulus is feeble or the intervening distance long or semi-conducting. Hence, under the above conditions, stimulus applied at a distance will give rise only to a positive response.
A reduction of the intervening distance will give rise to a different result. As the negative response is the more intense of the two, the feeble positive will be masked by the superposed negative. The separate exhibition of the two responses is only possible by a sufficient lag of the negative impulse behind the positive. This lag increases with increase of length of transmission and decreases with the diminution of the length. Hence the application of stimulus near the responding organ will give rise only to a negative response, in spite of the presence of the positive, which becomes masked by the predominant negative.[P]
These inferences have been fully borne out by results of experiments carried out with various specimens of plants under the action of diverse forms of stimuli. In all cases, application of stimulus at a distance causes a pure positive response; moderate reduction of the distance induces a diphasic response—a positive followed by a negative; further diminution of distance gives rise to a resultant negative response, the positive being masked by the predominant negative.
From what has been said it will be understood that the exhibition of positive response is favoured by the conditions, that the transmitting tissue should be semi-conducting, and the stimulus feeble. It is thus easier to exhibit the positive effect with the feebly conducting petiole of Averrhoa than with the better conducting petiole of Mimosa. It is, however, possible to obtain positive response in the Mimosa by application of indirect stimulus to the stem in which conduction is less rapid than in the petioles.
TABLE IX.—PERIODS OF TRANSMISSION OF POSITIVE AND NEGATIVE IMPULSES IN THE PETIOLE OF AVERRHOA AND STEM OF MIMOSA.
No.SpecimenDistance in mm.StimulusTransmission period for positive impulse.Transmission period for negative impulse.
1Averrhoa70Thermal22.0secs65 secs.
2"130 "40.0 "95 "
3"10Induction-shock 6.0 "20 "
4"20 "14.0 "48 "
5"35Chemical21.0 "50 "
6Mimosa5Induction-shock 0.5 "12 "
7"10 " 0.6 " 9.4 "
8"20 " 1.1 "10 "
9"60 " 2.0 "29 "
10"35Chemical 5.0 "17 "
EFFECTS OF DIRECT AND INDIRECT STIMULUS.
From the results given in course of the Paper we are able to formulate the following laws about the effects of Direct and Indirect Stimulus on pulvinated organs:—
1. Effect of all forms of Direct stimulus is a diminution of turgor, a contraction and a negative mechanical response.
2. Effect of Indirect stimulus is an increase of turgor, an expansion and a positive mechanical response.
3. Prolonged application of indirect stimulus of moderate intensity gives rise to a diphasic, positive mechanical response followed by the negative.
4. If the intervening tissue be highly conducting, the transmitted positive effect becomes masked by the predominant negative.
The laws of Effects of Direct and Indirect stimulus hold good not merely in the case of sensitive plants, but universally for all plants. This aspect of the subject will be treated in fuller detail in later Papers of this series.
IX.—MODIFYING INFLUENCE OF TONIC CONDITION ON RESPONSE
By
Sir J. C. Bose
Assisted by
Guruprasanna Das.
In experiments with different pulvinated organs, great difference is noticed as regards their excitability. If electric shock of increasing intensity from a secondary coil be passed through the pulvini of Mimosa, Neptunia, and Erythrina arranged in series, it would be found that Mimosa would be the first to respond; a nearer approach of the secondary coil to the primary would be necessary for Neptunia to show sign of excitation. Erythrina would require a far greater intensity of electric shock to induce excitatory movement. Organs of different plants may thus be arranged, according to their excitability, in a vertical series, the one at the top being the most excitable. The specific excitability of a given organ is different in different species.
In addition to this characteristic difference, an identical organ may, on account of favourable or unfavourable conditions, exhibit wide variation in excitability. Thus under favourable conditions of light, warmth and other factors, the excitability of an organ is greatly enhanced. In the absence of these favourable tonic conditions the excitability is depressed or even abolished. I shall, for convenience, distinguish the different tonic conditions of the plant as normal, hyper-tonic and sub-tonic. In the first case, stimulus of moderate intensity will induce excitation; in the second, the excitability being exceptionally high, very feeble stimulus will be found to precipitate excitatory reaction. But a tissue in a sub-tonic condition will require a very strong stimulus to bring about excitation. The excitability of an organ is thus determined by two factors: the specific excitability, and the tonic condition of the tissue.
THEORY OF ASSIMILATION AND DISSIMILATION.
A muscle contracts under stimulus; this is assumed to be due to some explosive chemical change which leaves the tissue in a condition less capable of functioning, or in a condition below par. Herring designates this as a process of dissimilation. The excitability of the muscle is restored after suitable periods of rest, by the opposite metabolic change of assimilation. “Assimilation and Dissimilation must be conceived as two closely interwoven processes, which constitute the metabolism (unknown to us in its intrinsic nature) of the living substance. Excitability diminishes in proportion with the duration of D-stimulus, or, as it is usually expressed, the substance fatigues itself. It is perfectly intelligible that a progressive fatigue and decrement of the magnitude of contraction must ensue. The only point that is difficult to elucidate is the initial staircase increment of the twitches, more especially in excised, bloodless muscle, which seems in direct contradiction with the previous theory.”[Q]
With reference to Herring’s theory given above, Bayliss in his “Principles of General Physiology” (1915), page 377 says, “In the phenomenon of metabolism, two processes must be distinguished, the building up of a complex system or substance of high potential energy, ‘anabolism,’ and the breaking down of such a system, ‘catabolism,’ giving off energy in other forms. The tendency of much recent work, however, is to throw doubt on the universality of this opposition of anabolism and catabolism as explanatory of physiological activity in general.”
The results obtained with the response of plants to stimulus may perhaps throw some light on the obscurities that surround the subject. They show that the two processes may be present simultaneously, and that the ‘down’ change induced by stimulus may, in certain instances, be more than compensated by the ‘up’ change.[R] I shall, for convenience, designate the physico-chemical modification, associated with the excitatory negative mechanical and electrical response of plants, as the “D” change; this is attended by run down of energy. The positive mechanical and electrical response must therefore connote opposite physico-chemical change, with increase of potential energy. This I shall designate as the “A” change, which by increasing the latent energy, enhances the functional activity of the tissue. That stimulus may give rise simultaneously to both A, and D, effects, finds strong support in the dual reactions exhibited in plant-response. Under indirect stimulus, the two responses are seen separately, the more intense negative following the feeble positive. When by the reduction of the intervening distance, stimulus is made direct, the resultant response, as previously stated, is negative; and this is due not to the total absence of the positive but to its being masked by the predominant negative. Let us next consider the question of unmasking this positive element in the resultant negative response.
UNMASKING OF THE POSITIVE EFFECT.
Under favourable conditions of the environment, the excitability of the organs is at its maximum. A given stimulus will bring about an intense excitation, and the ‘down’ D-change will therefore be very much greater than the A-change. Let us now consider the case at the opposite extreme where, owing to unfavourable condition, the excitability is at its lowest. Under stimulus the excitatory D-change will now be relatively feeble compared to the A-change, by which the potential energy of the system becomes increased. In such a case successive stimuli will increase the functional activity of the tissue, and bring about staircase response. Biedermann mentions the staircase response of excised bloodless muscle as offering difficulty of explanation. It is obvious that the physiological condition of the excised muscle must have fallen below par. The staircase response in such a tissue is thus explained from considerations that have just been adduced.
The results obtained with Mimosa not only corroborate them, but add incontestable proof of the simultaneous existence of both A and D changes. The physiological condition of a plant, Mimosa for example, is greatly modified by the favourable or unfavourable condition of the environment. In a hyper-tonic condition its excitability becomes very great; in this condition the plant responds to its maximum even under very feeble stimulus. Here the D-change is relatively great, and successive responses are apt to show sign of fatigue.
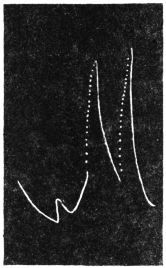
Fig. 53.—Record showing the effect of stimulus modifying tonicity and producing staircase effect. (Mimosa)
But the plant in a sub-tonic condition will exhibit feeble or no excitation. The D-change will be absent while the A-change will take place under the action of stimulus. This, by increasing the potential energy, will enhance the functional activity of the tissue.
Staircase response in Mimosa: Experiment 48.—The theoretical considerations will be found experimentally verified in the record obtained with a specimen of Mimosa in a sub-tonic condition (Fig. 53). Owing to the lack of favourable ‘tone’ the leaf was relaxing as seen in the first part of the curve. The stimulus of electric shock, applied at the thick dot in the curve slanting downwards, gave no response but raised the tone of the tissue by arresting the growing relaxation. Subsequent stimuli gave rise to staircase responses. Stimulus has, through the A-effect, raised the functional activity of the tissue to a maximum.